Tag Archives: Nature conservation

Bees, moths, cockroaches and some unfortunate flies: the surprising pollination of a European milkweed

Back in October 2021, I wrote a post about tracking down a rather elusive plant on the Danish coast. Karin and I had been cycling around the Odsherred region when I spotted the distinctive yellowing autumn foliage of Vincetoxicum hirundinaria growing close to the little fishing harbour at Klint.

I was particularly pleased to find it because Vincetoxicum is a genus of plants that I’ve been interested in for many years. It’s part of the milkweed and dogbane family, Apocynaceae, and belongs to the subfamily Asclepiadoideae, a group with some of the most extraordinarily complex flowers in the plant kingdom.

At the end of that post I asked a question: what was pollinating those flowers on the exposed Danish shoreline? At the time there were surprisingly few published records of pollinators for this widespread European species.

Five years later, I’m delighted to say that a new paper just published in AoB PLANTS, led by my Chinese colleague Wujian Xiong, and to which I’ve contributed, goes a considerable way towards answering that question. Not specifically for the Danish population, but for several populations studied in and around Salzburg, Austria. And the answer is rather more complicated, and interesting, than we might have expected.

A very specialised flower with remarkably unspecialised tastes

The flowers of Vincetoxicum hirundinaria are small, pale cream or ivory-coloured, and about 12 mm across. Like other members of the Asclepiadoideae, they have a highly specialised mechanism for transferring pollen.

Rather than producing individual loose pollen grains, the pollen is packaged into structures called pollinia, which are joined together by a central attachment mechanism to form a pollinarium. When an insect visits a flower, part of its body can become caught in a narrow guiding structure. As it pulls away, a pollinarium may become attached to its mouthparts, legs or other appendages. If all goes well, the insect carries that pollen to another flower and deposits it into a specialised receptive chamber.

It’s an extraordinarily precise mechanism, and one might reasonably expect that only a rather narrow range of insects could operate it successfully.But that’s not what we found.

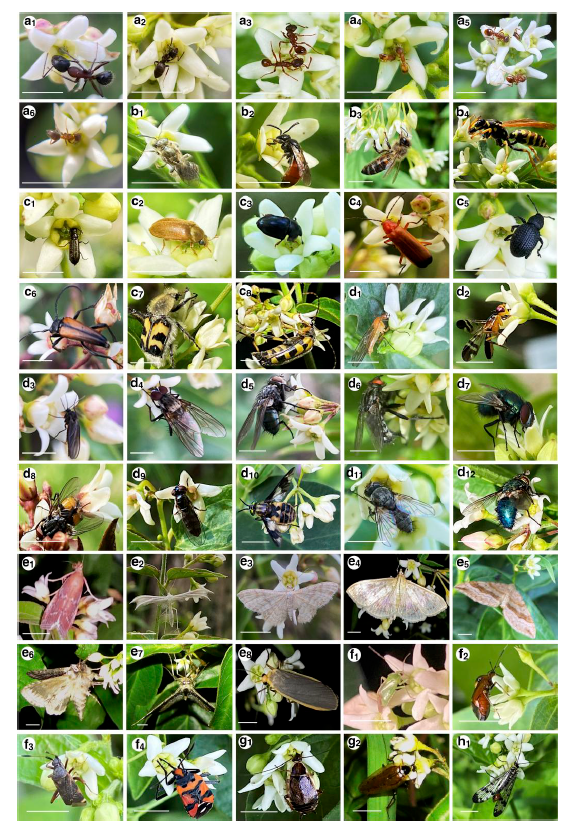
Over 50 hours of observations, Wujian recorded almost 3,000 visits to the flowers, involving 81 species or morphospecies of insects from seven different orders. These included bees, wasps, ants, flies, beetles, moths, bugs, scorpionflies and cockroaches.

Of those 81 types of flower visitor, 37, representing five insect orders, were found carrying pollinaria. These included 15 types of flies, seven bees and wasps, seven moths, six ants, one beetle and one cockroach. That’s a remarkably diverse assemblage for a plant with such specialised floral structures. Indeed, it’s the most diverse pollinator assemblage so far documented for any member of Vincetoxicum.

What makes this particularly interesting is that the pollinaria were attached to different parts of the insects’ bodies. In flies they might be on the proboscis or legs; in bees and wasps on the mouthparts; in moths on the proboscis; and in cockroaches on the labial palps.

In other words, the same elaborate floral mechanism can operate with insects that differ enormously in their anatomy, size and behaviour.

Another chapter in the story of cockroach pollination

There’s a particularly satisfying connection here with another paper that Wujian and I published back in 2020. That study demonstrated specialised cockroach pollination in the rare and endangered Chinese species Vincetoxicum hainanense. Its small flowers open at night, produce an unpleasant scent reminiscent of rotting fruit, and are principally pollinated by a particular species of cockroach, Blattella bisignata.

It was the first documented example of specialised cockroach pollination in the Apocynaceae, and one of only a handful of well-studied examples from anywhere in the world. Now we have another species of Vincetoxicum that is visited and potentially pollinated by cockroaches, but in this case they are just one component of a much more diverse assemblage.

The contrast between the two species is striking. They share the same basic type of highly specialised floral architecture, yet one has a relatively narrow pollination system while the other is much more generalised. Clearly, floral complexity doesn’t necessarily translate into ecological specialisation.

Day and night, and the importance of place

Another interesting finding concerns when the flowers are available to pollinators. The flowers of V. hirundinaria open in the late afternoon, between about 4pm and 6pm, and remain open for an average of six days. They produce nectar and a strong, sweet scent that we describe in the paper as reminiscent of red wine.

That long floral lifespan means that they are potentially accessible to both daytime and nocturnal insects. But the relative importance of those insects varied considerably between the study populations. At most sites, pollen removal and deposition took place during the day, with bees, wasps and other diurnal insects playing the main roles. However, at the higher-elevation Gaisberg site, nocturnal moths and cockroaches were much more prominent, and pollen transfer during the night was particularly effective.

It’s a useful reminder that a plant doesn’t necessarily have one fixed set of pollinators across its geographical range. The animals available to visit flowers can change with location, habitat, season and time of day. This connects with some of the arguments that I’ve made recently about geographical variation in plant–pollinator specialisation. Ecological specialisation isn’t always an intrinsic, unchanging characteristic of a species, it can depend very much on the circumstances in which that species is studied.

But not every visitor is a useful pollinator

There’s a rather darker side to this story, however: the flowers of Vincetoxicum hirundinaria can be surprisingly dangerous places for small insects. We recorded 16 types of flies that became trapped by the flowers, often fatally, when their mouthparts became lodged in the structures associated with the pollinarium. Some were simply too small or weak to pull themselves free.

This phenomenon is known from other milkweeds, including the notorious moth-catching vine Araujia sericifera. However, the extent of insect trapping that we observed in V. hirundinaria was quite remarkable. There’s an important distinction here between attracting an insect to a flower and actually using it to transfer pollen successfully, even for those species that don’t get trapped.

Ants, for example, accounted for about a quarter of all recorded flower visits, but only 3.5% of the sampled ants carried pollinaria. In contrast, between 40% and 60% of individuals in several other insect groups carried pollinaria.

Even carrying a pollinarium doesn’t necessarily mean that an insect will successfully deposit pollen into another flower. That requires the insect to visit a suitable flower and position its body in just the right way. I’ve discussed this issue before in relation to what we actually mean by a pollination system. Counting floral visitors is relatively straightforward. Demonstrating that those visitors contribute to successful plant reproduction is much more difficult.

In the present study, the evidence for functional generalisation is strong in terms of the diverse insect groups capable of removing and transporting pollinaria. However, we cannot yet say precisely how much each group contributes to successful pollen deposition and seed production.

Indeed, overall pollen transfer efficiency was quite low. At most sites only about 3–9% of the pollen removed from flowers was successfully transferred to another flower’s receptive structures during the day. At Gaisberg, nocturnal pollen transfer efficiency averaged around 11%. Nor did the plants produce many fruits. Only 2% of naturally pollinated flowers produced mature fruits, compared with 14% following experimental cross-pollination. The plants were also self-incompatible in the populations we studied, meaning that pollen transferred between flowers of the same individual wouldn’t result in successful reproduction.

So despite attracting a remarkably diverse range of insects, V. hirundinaria appears to have substantial limitations on its reproductive success. Pollination isn’t simply a numbers game.

Back to the bigger picture

Readers of this blog will know that the diversity and evolution of pollination systems in Apocynaceae has been a major theme of my research for many years. In our large international review published in 2019, we brought together information on the pollinators of 567 species and showed that the family encompasses everything from extremely specialised relationships to highly generalised systems involving many different kinds of animals.

More recently, I’ve written about the extraordinary pollination biology of Heterostemma ficoides, which deceives fig wasps while providing genuine breeding opportunities for tiny flies. And only last week I discussed our new study of eleven co-occurring Apocynaceae species in Argentina, showing how very different flowers can share overlapping assemblages of visitors.

The new Vincetoxicum study adds another piece to this evolutionary and ecological puzzle. It demonstrates that even one of the most mechanically sophisticated types of flower can function with a very wide range of potential pollinators. Floral specialisation and pollinator specialisation are not the same thing, and we shouldn’t assume that one necessarily predicts the other.

But it also raises some intriguing questions. Why do the flowers attract so many insects that seem poorly suited to pollinating them? Is this simply an unavoidable consequence of producing nectar and scent signals that appeal to many different animals? Or might the presence of trapped insects actually reduce reproductive success by blocking access to the flowers’ reproductive structures?

And, returning to where I started, what exactly is pollinating those plants on the Danish shoreline at Klint? Are they visited by the same diversity of insects as the Austrian populations, or has their rather exposed coastal environment resulted in a very different assemblage? I still don’t know the answer to that question. But it would be fascinating to find out.

One of the things I enjoy most about working on the Apocynaceae is that each new study seems to reveal another layer of complexity in this extraordinary family. Almost 40 years after I began studying their flowers and pollinators, they continue to surprise me. My thanks to Wujian and all of our colleagues for helping to unravel another part of that story.

Here’s the full reference, with a link to the open-access paper:

Xiong, W., Ollerton, J., Liede-Schumann, S., Meve, U., Wagner, H.C., You, W., Mu, J. & Dötterl, S. (2026) Generalized pollination of morphologically specialized Vincetoxicum hirundinaria (Apocynaceae, Asclepiadoideae). AoB PLANTS 18(5): plag048. https://doi.org/10.1093/aobpla/plag048

Images above (c) Wujian Xiong
Moths, wasps, hummingbirds and nectar: exploring the pollination ecology of Apocynaceae in Argentina

One of the things that has fascinated me throughout my career is the extraordinary diversity of ways in which flowering plants interact with their animal visitors. Nowhere is this better illustrated than in the milkweed and dogbane family, the Apocynaceae, a group that I’ve been studying for almost 40 years.

Only last month I wrote about the remarkable pollination biology of Heterostemma ficoides, a species from Thailand that deceives fig wasps while offering a genuine breeding site to tiny flies. That was an example of an unusual pollination system involving a single species. But what happens when we look at a whole community of Apocynaceae growing together in the same habitat? Do they share pollinators, or have they evolved different ways of attracting and using animals?

Those are some of the questions that my Argentinian colleagues Carolina Torres and Leonardo Galetto and I have addressed in a new paper just published in the journal Taxon. The study focuses on eleven species of Apocynaceae growing together in the Chaco forests of central Argentina, a region characterised by strongly seasonal rainfall and a distinctive assemblage of plants and animals.

What’s particularly interesting is that the original field observations were made by Carolina and Leonardo over three flowering seasons between 1997 and 2000. We have now brought those data together, including detailed measurements of floral nectar, and added analyses of the networks of interactions between plants and their visitors. It’s a nice example of how carefully collected field data can continue to yield new insights many years later.

Different flowers, different rewards

The eleven species represent three major evolutionary lineages within the Apocynaceae: one rauvolfioid, three apocynoids (Mandevilla species), and seven members of the Asclepiadoideae, the group formerly recognised as the separate family Asclepiadaceae.

Their flowers vary enormously in size and structure. At one extreme are the relatively small flowers of species such as Araujia, Oxypetalum and Philibertia. At the other are the large, tubular flowers of Mandevilla, including M. petraea, in which the functional floral tube is more than 10 cm long.

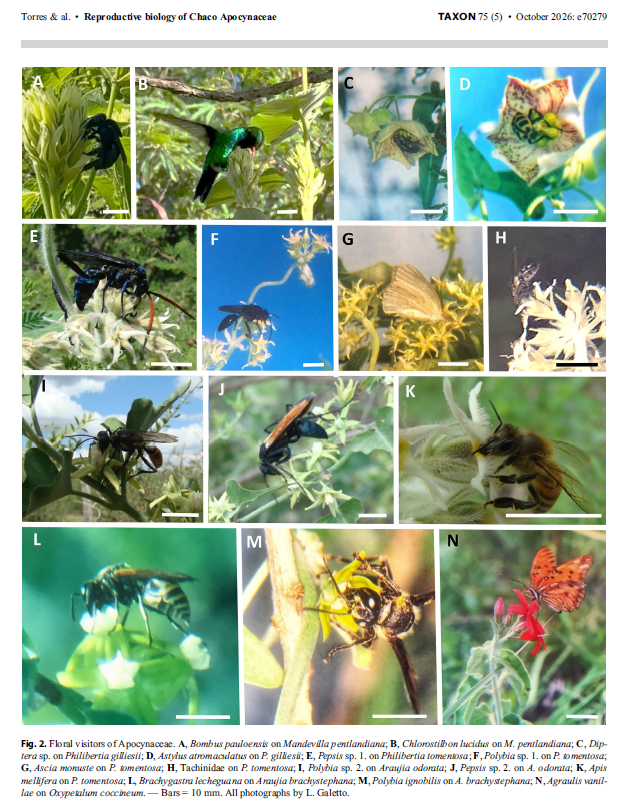
These differences are reflected in the nectar that the flowers produce. The three Mandevilla species generally offer relatively large quantities of nectar containing substantial amounts of sugar, predominantly sucrose. They are visited by animals capable of accessing these rewards, including long-tongued hawkmoths, bumblebees and, in the case of M. pentlandiana, hummingbirds. By contrast, most of the smaller-flowered species produce much less nectar and show greater variation in the proportions of the three main nectar sugars: sucrose, glucose and fructose.

But these relationships are not quite as straightforward as we might expect. For example, two closely related species, Araujia brachystephana and A. odorata, have rather similar-looking flowers, yet the former produces nectar dominated by sucrose while the latter produces nectar consisting almost entirely of glucose and fructose. Both are visited primarily by wasps, although A. brachystephana attracts a broader range of insects.

In other words, even closely related species living in the same habitat may differ substantially in the rewards they offer and the animals that visit them.

There’s another intriguing result concerning the tree Aspidosperma quebracho-blanco. Previous research described its flowers as deceptive, attracting visitors without offering nectar. Yet in our study we found small quantities of nectar containing mainly glucose and fructose. Does nectar production vary between populations, or were there differences in the methods used to study the flowers? It’s an interesting question that deserves further investigation.

Sharing the flowering season

The timing of flowering is another important part of this ecological story. Most of the species flowered during the warmer, wetter months, particularly December and January, with flowering often continuing for three or four months. Seed dispersal, by contrast, was concentrated mainly between February and June, when conditions become progressively drier.

This makes ecological sense. Water availability is likely to be an important trigger for flowering in this seasonal environment, while the wind-dispersed seeds of these species are released mainly during the drier part of the year. But it also means that many of the species are flowering simultaneously and potentially competing for the attention of the same animals.

One possibility is that plants avoid this competition through differences in flowering time. Another is that they coexist by attracting different groups of pollinators, or by using the same pollinators in subtly different ways. For example, two Mandevilla species may share hawkmoth visitors but place their pollen on different parts of the moth’s proboscis, potentially reducing interference between their reproductive systems.

Among the smaller-flowered asclepiads, differences in the intricate structures that attach pollen masses to visiting insects may perform a similar function. These are fascinating examples of how floral morphology can influence ecological interactions, even when the same animals visit several plant species.

What do the interaction networks tell us?

As readers of this blog will know, I’ve been interested in plant–pollinator networks for many years. One reason for analysing these networks is that they allow us to move beyond individual plant species and examine how an entire assemblage of organisms is connected.

In the Chaco study, we found a mixture of apparently specialised and generalised relationships. Some species were visited by just one major functional group, such as wasps or butterflies, while others attracted a much wider range of insects. Wasps were particularly conspicuous. Indeed, two social wasps, Polybia ignobilis and Brachygastra lecheguana, were among the visitors that connected different parts of the interaction network. The introduced western honey bee, Apis mellifera, also played a connecting role.

It’s another reminder that when we talk about pollinators, we really need to look beyond bees. Wasps, flies, moths, butterflies and other animals can be important components of these ecological communities.

One intriguing outcome of our analyses concerns the overall structure of the network. At first glance, the interactions appear to be organised into distinct groups, or modules, with particular sets of plants sharing particular sets of visitors. However, when we compared the observed network with randomly generated networks that preserved the number of interaction partners of each species, neither its modularity nor its nestedness was significantly greater than expected.

In other words, although some groups of interactions look rather specialised, there is limited statistical evidence for strong compartmentalisation within this particular assemblage. The patterns may largely reflect differences in how many partners each species has, rather than the existence of clearly separated ecological groups.

There is an important qualification here. Our network includes only eleven plant species, all from the same family, rather than the full diversity of flowering plants in the Chaco forests. A more comprehensive network might reveal additional structure that we cannot detect at this scale.

This connects rather neatly with my recent discussion of global patterns in plant–pollinator specialisation. One of the lessons from that research is that specialisation depends partly on the spatial, taxonomic and ecological scale at which interactions are examined. What looks specialised at one scale may be much more generalised at another.

I should also emphasise that this is a network of floral visitors, not necessarily effective pollinators. We recorded animals capable of contacting the reproductive structures of the flowers, and of carrying pollinaria, but that does not establish that they successfully transferred pollen between plants. As I discussed in an earlier post about what we actually mean by a pollination system, that distinction really matters.

Back to the bigger picture

For me, this study makes an interesting contribution to the broader understanding of Apocynaceae pollination ecology that my colleagues and I developed in our 2019 global review of the family’s pollination systems. In that paper, involving 75 authors, we showed that Apocynaceae exhibit an extraordinary diversity of pollination systems, with strong evolutionary and biogeographical patterns. But we also emphasised how much remains unknown, with reliable pollination information available for only a little over 10% of the family’s species. The new Chaco study adds something that large-scale reviews cannot provide on their own: a detailed picture of how related species interact with their floral visitors within the same ecological community.

There’s also a connection to our recent review of edible Apocynaceae, which also involved Carolina and Leonardo. One of the striking results of that study was how little we know about the pollination biology of many species whose fruits, seeds or other parts are used by people. Understanding how these plants reproduce is important not only from an evolutionary perspective but also for their conservation and sustainable use.

Ultimately, what I find most interesting about this new paper is the contrast between the extraordinary diversity of floral forms and rewards, and the extent to which different species can share the same visitors. Specialised flowers do not necessarily mean exclusive relationships with particular pollinators. And generalised patterns of visitation do not mean that floral morphology and nectar chemistry are unimportant. The reality is more complicated, shaped by evolutionary history, seasonality, floral structure and the behaviour of the animals themselves.

It’s also a reminder of the continuing value of detailed natural history. Large-scale databases and sophisticated network analyses are enormously useful, but they depend ultimately on people spending time in the field, watching what visits flowers, measuring nectar, and recording when plants flower and produce seeds. Sometimes those observations take decades to reach their full potential. But that doesn’t make them any less valuable.

Here’s the full reference, with a link to the paper:

Torres, C., Ollerton, J. & Galetto, L. (2026) Reproductive phenology, flower-nectar traits, and floral visitors of eleven co-occurring species of Apocynaceae from Chaco forests (Argentina). Taxon 75(5): e70279. https://doi.org/10.1002/tax.70279

Are plant-pollinator interactions more specialised in the tropics? A new global analysis suggests that it’s complicated…

Some scientific questions have a habit of following you around for much of your career. Back in 2002, Louise Cranmer and I published a paper in the journal Oikos asking a deceptively simple question: are tropical plants more specialised in terms of their pollinators?

At the time there was a widespread assumption in ecology that interactions between species become increasingly specialised as you move from the poles towards the tropics. It’s an attractive idea which had some (quite vague) theoretical support. Tropical ecosystems contain more species, have experienced relatively stable climates over long periods of evolutionary time, and seem like just the sort of places where tightly specialised interactions ought to evolve.

The trouble was that the evidence wasn’t especially convincing, in part because it hadn’t actually been well studied. In preparing the 2002 paper, Louise and I found only a handful of empirical studies that had addressed the question, not just for plants and pollinators, but for ALL kinds of interactions.

The question of tropical specialisation has subsequently cropped up repeatedly in my research. In 2014, Angela Moles and I went considerably further and asked whether the broader claim that species interactions are stronger and more specialised in the tropics might actually be a “zombie idea” – one of those scientific notions that persists despite accumulating evidence that the reality is considerably more complicated. That guest post on the Dynamic Ecology blog was then written up as an invited paper for Biotropica see: Tropical Zombies: Moles & Ollerton (2016) is now published.

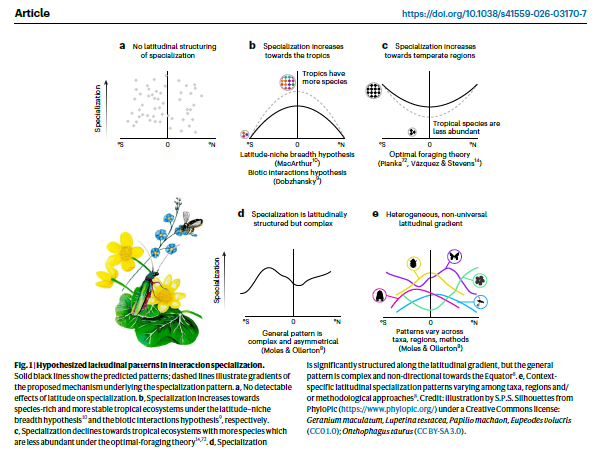
Twenty-four years after that first Oikos paper, we can now address the question with a dataset that Louise and I could scarcely have imagined in 2002. A huge international collaboration led by Sailee Sakhalkar and Robert Tropek has just published “Global patterns in plant–pollinator specialization” in Nature Ecology & Evolution.

I’m delighted to be one of the co-authors and I find the answer to the question that we posed 24 years ago to be fascinating.

More than 110,000 interactions

The scale of the new study is worth emphasising. It assembled 3,415 quantitative plant-pollinator networks from 162 studies, covering 110,571 pairwise interactions between 5,343 pollinator species and 6,126 plant species. The data span almost all of the world’s terrestrial biogeographic regions, from 43.6°S to 81°N and from sea level to more than 4,000 metres elevation.

That makes this the most comprehensive attempt yet to examine the geography of specialisation in plant-pollinator interactions. But simply throwing thousands of networks into a statistical analysis would potentially create as many problems as it solves. Different researchers study pollination networks in very different ways. Some attempt to sample whole communities, while others concentrate on particular groups such as bees, hummingbirds or particular plants.

So an important feature of this study was that we explicitly separated these different types of datasets and accounted for sampling completeness and methodological differences. We also looked separately at different functional groups of pollinators rather than assuming that bees, beetles, butterflies, moths, flies and birds should all behave in the same way. That turned out to be important in ways that we could not predict.

So, are interactions more specialised in the tropics?

The short answer is no, not in any simple sense. There is geographical structure to plant-pollinator specialisation. But there is no straightforward increase in specialisation as you approach the Equator – nor, for that matter, a straightforward decrease. Instead, the patterns are distinctly nonlinear.

Network-level specialisation and pollinator specialisation tended to peak at relatively low northern latitudes, at around 20°–30°N, close to the tropical-subtropical boundary. I find this particularly interesting as I think the subtropics have been a bit neglected as a focus of ecological research: no one ever refers to themselves as a “subtropical ecologist” and there is no Journal of Subtropical Ecology. Yet the subtropics are not simply a transitional zone between the tropical and temperate worlds. They encompass an extraordinary range of ecosystems, including deserts, Mediterranean-type vegetation, subtropical forests, and some major centres of biodiversity and endemism. This includes the distinctive habitats in Yunnan that I’m exploring during my visits to China. Perhaps we need to start thinking of the subtropics as an important biogeographical region in their own right, rather than as the ecological space between two better-studied zones?

Plant specialisation showed a different and weak hemispherically asymmetric pattern. And once individual pollinator groups were examined separately, the picture became more complicated still. Hoverflies, for example, came closest to the traditional expectation of increasing specialisation towards the Equator. Birds showed something closer to the opposite pattern, while moths did something much more complicated.

In other words, there isn’t a latitudinal specialisation gradient. There are several overlapping geographical patterns whose shapes depend upon what organisms you study and what measure of specialisation you are considering.

That conclusion feels satisfying given the arguments Angela Moles and I made ten years ago. We suggested that attempts to find a universal latitudinal gradient could obscure the fact that different groups of organisms have different evolutionary histories, physiologies and ecologies. That is very close to what emerges from this much larger analysis.

Perhaps latitude was never really the interesting variable

One of the most intriguing results is what happens when we stop asking about latitude itself. We compared latitude with a suite of possible explanatory variables, including temperature, precipitation, environmental productivity, and plant and pollinator diversity. Climate generally did a better job of explaining specialisation than latitude, biodiversity or productivity. Again, however, there wasn’t a single climatic rule.

At the whole-network level, specialisation generally declined as mean annual temperature increased, which was not expected at all and runs counter to the argument that the tropics are always more specialised. Precipitation produced strongly nonlinear relationships, and plants and different pollinator groups responded differently. Birds, insects and even different groups of insects could show contrasting responses to the same climatic gradient.

There are some plausible biological explanations for these patterns. Warmer conditions may extend flowering periods and pollinator activity, creating more opportunities for species to encounter alternative partners and therefore encouraging generalisation. Colder or more seasonal environments might compress flowering and pollinator activity into shorter periods, producing tighter temporal matching between species. Rainfall adds another layer of complexity because it can influence flowering but also directly constrain pollinator activity.

These are hypotheses rather than demonstrated mechanisms, however. As we stress in the paper, these are correlational global patterns and climate covaries strongly with latitude. The results shouldn’t therefore be interpreted as demonstrating simple causal effects of temperature or rainfall.

Specialisation depends on how you look at it

There’s another connection here to research I’ve discussed previously on the blog. In work with Danish and Brazilian colleagues, for example, we showed that the apparent specialisation of plants and pollinators depends partly on the spatial scale at which interactions are examined – see Local and regional specialization in plant–pollinator networks. More recently I’ve written about why scale matters when analysing plant-pollinator networks.

And earlier this year, our global analysis of plant-pollinator interactions in gardens found that the factors explaining species richness were not necessarily those explaining interaction specialisation: Global drivers of plant-pollinator interaction specialization in gardens.

There’s also a nice connection to another study that I wrote about here in 2022. With Pablo Gorostiague and Pablo Ortega-Baes, I looked specifically at whether cactus pollination systems become more specialised towards the tropics. Our answer was yes and no: tropical cacti were visited by somewhat fewer pollinator species, but there was no latitudinal pattern in the number of functional pollinator groups that they used. As I wrote at the time, the answer depended on what we meant by “specialised”: Are cactus pollination systems more specialised in the tropics? A new study suggests yes…and no!

All of these studies point towards a similar conclusion: “specialisation” is not a single, fixed property of an ecological community. What we detect depends upon biological scale, geographical scale, the organisms being considered, and how the interactions have been sampled. That doesn’t make specialisation meaningless. Quite the opposite, it means we need to be precise about what sort of specialisation we’re talking about and at what scale.

The new global study puts that result into a much broader context. Different groups really can display different geographical patterns of specialisation, so studies focused on a particular lineage aren’t necessarily contradicting one another when they produce different answers. They may simply be measuring different pieces of a much larger ecological puzzle.

Why does any of this matter?

Specialisation is not just an esoteric property of ecological networks. It affects how plants and pollinators partition resources, how species coexist, how communities are assembled, and potentially how ecological systems respond when species disappear.

That becomes especially important in a changing climate. Our results suggest that changing temperature and rainfall regimes could restructure plant-pollinator networks, but they are unlikely to do so uniformly. Different pollinator groups and different parts of the world may respond in very different ways. Highly specialised interactions may also be particularly vulnerable to changes in phenology or the loss of interaction partners. Predicting the consequences therefore requires us to move beyond simple statements about “tropical” and “temperate” ecosystems.

For me, though, there is also a broader lesson here about how science progresses. In 2002, Louise Cranmer and I questioned whether the available evidence really supported the assumption that tropical plant-pollinator interactions were more specialised. Fourteen years later, Angela Moles and I argued that the wider claim about stronger and more specialised tropical interactions might be a zombie idea. Now, with more than 110,000 plant-pollinator interactions available for analysis, the answer is much clearer. Latitude matters; climate matters; the identity of the organisms matters; and ecology, as usual, refuses to obey a simple rule.

My particular thanks to Sailee and Rob for the monumental efforts they made to pull this work together, and cudos to all of the co-authors who helped to make the study possible.

A century of genetic erosion in a British bumblebee – a new study just published

Back in 2022 I wrote about a project in which I’d been involved with colleagues at the Natural History Museum, Imperial College London and several regional museums. We were using preserved bumblebees to ask a deceptively simple question: what can insects collected decades ago tell us about the environmental changes that their populations have experienced?

The first papers from that project showed two important things. One found increasing signs of developmental stress in the wings of museum bumblebees over the course of the 20th century, associated particularly with hotter and wetter conditions. The other demonstrated that it was possible to recover and sequence surprisingly good-quality DNA from insects collected more than a century ago, in some cases using just a single leg.

At the time I wrote that this opened up the possibility of looking at how the genomes of bee populations had changed through time. Well, we’ve now done it.

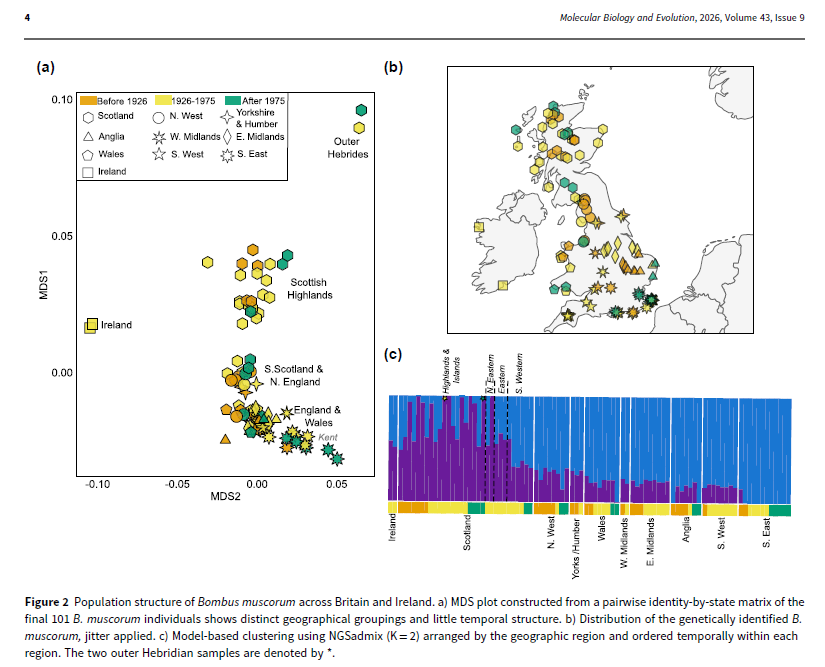
Published this week in Molecular Biology and Evolution, our new study focuses on the Moss Carder Bumblebee (Bombus muscorum), a beautiful species of flower-rich grasslands, heaths, marshes and coastal habitats. Once much more widespread across Britain, it is now largely concentrated in Scotland and the Scottish islands, with scattered populations surviving around the coasts of England and Wales.

Led by Victoria Mullin, the team generated whole-genome data from museum specimens collected between 1894 and 2019. The results provide a rather sobering picture of what has happened inside these bee populations as their geographical distribution has contracted.

Comparing bees collected before 1926 with those collected after 1975, we found about a 25% reduction in genome-wide genetic diversity. Looking at the full time series gives the same basic message: heterozygosity declined progressively through the 20th century, with no obvious sign of recovery.

That matters because losing a species is not the only way that biodiversity can decline. Long before extinction, populations can become smaller and more isolated and begin to lose genetic variation. That variation is part of the raw material that allows populations to respond to environmental change, disease and other challenges.

There was also a striking geographical pattern. In England and Wales, the amount of the genome occurring in long stretches of homozygosity increased by about 186% – in other words, almost threefold. These “runs of homozygosity” are consistent with populations becoming smaller, more fragmented and increasingly isolated from one another. Scotland showed a much weaker change, reflecting the fact that B. muscorum remains considerably more widespread there.

Importantly, however, the population structure is not simply “Scottish bees versus English bees”. The genomic data reveal a broad north-to-south gradient across Britain – what population geneticists call isolation by distance – rather than a set of sharply separated populations. That has implications for conservation because fragmentation may be breaking what was once a more continuously connected population into increasingly isolated regional groups.

There’s another interesting connection here with work that I published with colleagues more than a decade ago. In our 2014 Science paper we used historical records to show that Britain had lost 23 species of bees and flower-visiting wasps, with the fastest rate of extinction occurring from roughly the late 1920s to the late 1950s. We argued that large-scale changes in British agriculture, beginning just after the First World War, were an important part of that story.

The new study is looking at genetic change within a surviving species rather than the disappearance of whole species and it cannot pin that change on a single cause. But the parallels are difficult to ignore. The loss and fragmentation of flower-rich habitats associated with agricultural intensification is a likely contributor, alongside pesticides, climate change and other environmental pressures. The genomic erosion appears to have accumulated progressively across much of the same century in which Britain’s pollinator landscapes were being radically transformed.

One unexpected finding was also a useful warning about museum data. Of the 130 specimens originally labelled as Bombus muscorum, genetic analysis showed that 29 (almost a quarter) were actually two other, morphologically similar bumblebee species. Museum collections are extraordinarily valuable, but identifications cannot always simply be taken at face value, particularly for difficult groups. Genomics provides both a historical record and a way of checking the identity of the specimens supplying that record.

And that brings me back to what I think is one of the wider messages of this whole project: natural history collections are not dusty archives of dead organisms, they are biological time series.

A pinned bumblebee collected more than a century ago preserves information about where a species occurred, what environmental stresses it experienced, and, as we can now show, the genetic diversity of the population from which it came. Combined with modern genomic techniques, the millions of insects sitting in museum drawers around the world represent an extraordinary resource for understanding biological change.

The conservation message for the Moss Carder Bumblebee itself is fairly straightforward. Protecting the remaining populations is not enough if they become progressively smaller and more isolated. Restoring large areas of suitable, flower-rich habitat and reconnecting populations should help maintain population sizes and gene flow. More interventionist approaches such as translocation or assisted gene flow may eventually have a role, but would need careful assessment because of issues such as local genetic structure and disease transmission.

Four years ago, when I blogged about the first papers from this project, I finished with the idea that museum genomics might allow us to understand how insect populations had adapted, or failed to adapt, to a century of environmental change. We now have part of that answer. And it shows that beneath the visible contraction of a species’ range, another quieter form of biodiversity loss can be taking place: the erosion of diversity within its genome.

The paper is open access and you can download a copy here:

Mullin, V.E., Merchant, H.N., Arce, A.N., Nash, W. et al. (2026) Museum specimens reveal the genomic consequences of long-term population decline in an insect pollinator. Molecular Biology and Evolution 43: 1-11.

Nature and national security: some recent developments

Back in January I wrote a post entitled Pollination as a matter of national security, prompted by the UK Government’s rather extraordinary publication of this report: Global biodiversity loss, ecosystem collapse and national security: a national security assessment. My argument was that although pollination is obviously not a national security issue in the traditional sense of defending a country against hostile states or terrorist attacks, the loss of pollinators threatens food production, supply chains and the functioning of ecosystems upon which societies ultimately depend. In other words, it is a threat to national resilience, which we can define a country’s capacity to anticipate, withstand, adapt to, and recover from major shocks or long-term pressures while maintaining the essential functions of society, the economy, government, and critical infrastructure. I’ll come back to this national-level framing at the end.

I concluded that post by suggesting that the real question was not whether pollination could be regarded as a national security issue, but whether national security thinking had fully adapted to the biological foundations on which societies depend.

Since January, several reports, papers and policy developments have convinced me that this is becoming a much wider and more serious discussion. Pollination is only one component of it. What is emerging is a view of nature itself as part of the infrastructure that makes societies secure.

Nature as infrastructure

Perhaps the clearest expression of this idea comes from a paper by Bradley Cardinale, Emmett Duffy and Rod Schoonover entitled Nature’s role in national security, published this summer in the journal Nature-Based Solutions.

The authors consider five areas where ecological disruption can generate national security risks: food security, water scarcity, health security, protection from natural disasters, and environmental crime. In each case, environmental degradation can create or amplify economic and social pressures which, under some circumstances, translate into political instability and security problems.

What I particularly like about the paper is its use of the term “natural infrastructure”. Functioning ecosystems, the authors argue, operate rather like electricity grids, communications systems and transport networks. They provide services and, crucially, buffer societies against shocks.

This is an important shift in emphasis. We usually talk about the benefits or ecosystem services that nature provides. Both are perfectly useful concepts, but describing ecosystems as infrastructure changes how we think about their loss. A degraded wetland is then not simply a conservation problem. It may represent the deterioration of flood-control infrastructure. Similarly, a damaged watershed is a weakening of water-security infrastructure, whilst a decline in pollinators can be understood as damage to parts of our food-production infrastructure.

Seen in that way, restoring ecosystems begins to look less like discretionary environmental spending and more like preventive investment in resilience.

Rewilding as defence

An even more striking example appeared in April in The RUSI Journal, published by the Royal United Services Institute, one of the world’s oldest defence and security think tanks.

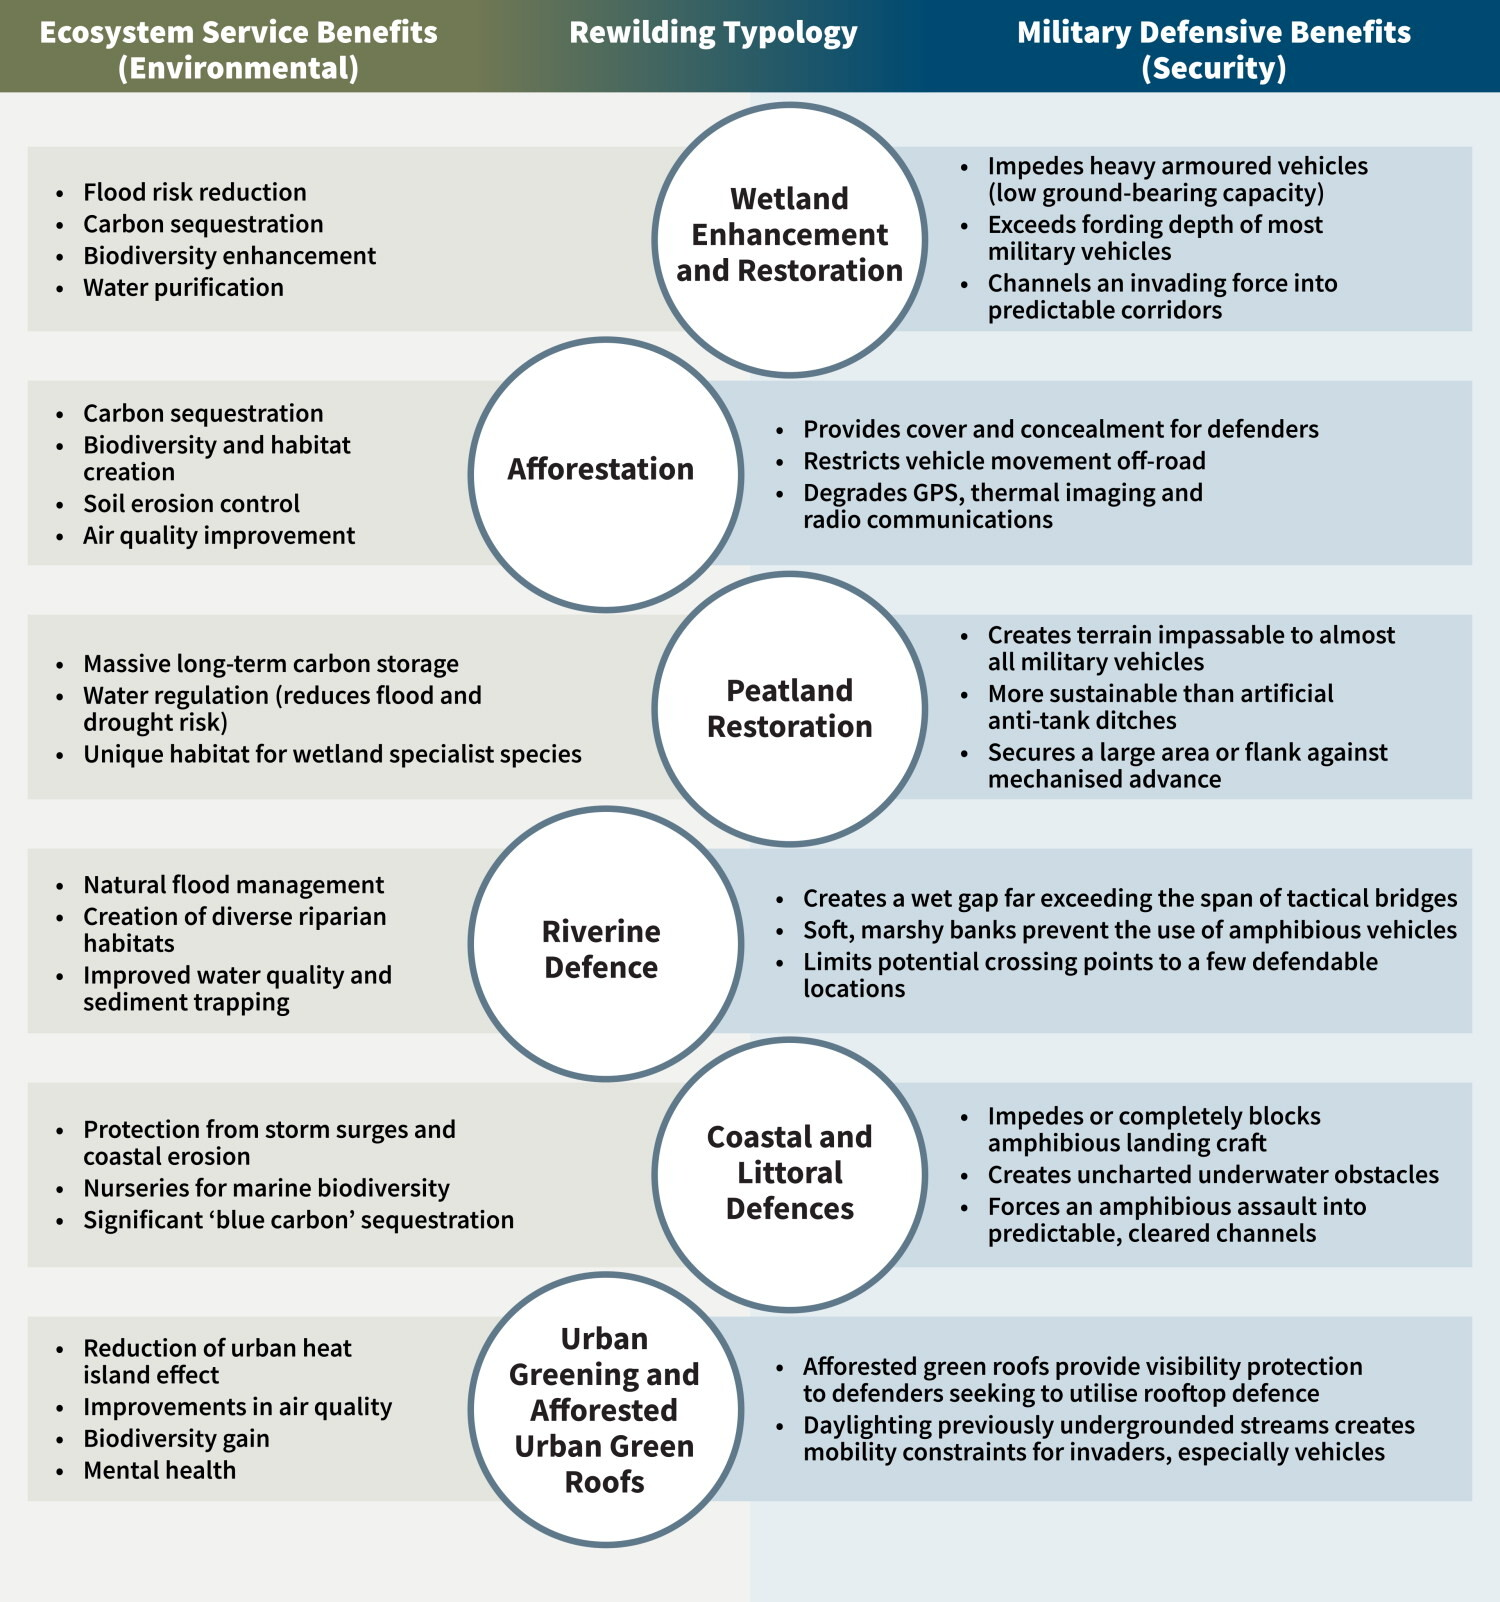
Sam Jelliman, Brian Schmidt and Alan Chandler propose the concept of “defensive rewilding”: strategically restoring forests, wetlands, peatlands and other ecosystems in locations where they could also impede, divert or slow an invading military force. This infographic from the paper outlines their argument quite persuasively:

At first sight this sounds rather eccentric, but the logic is straightforward. Military planners since at least the time of Alexander the Great have always understood that terrain matters. At the Battle of Issus in 333 BCE, for example, Alexander fought the much larger Persian army on a narrow strip of land between the sea and the mountains, restricting its ability to manoeuvre and helping to neutralise its numerical advantage. Wetlands, forests, rivers, hedgerows and boggy ground can also provide advantage by restricting visibility and movement and make the passage of vehicles and troops much more difficult. We have seen examples of this during the war in Ukraine, just as we did in numerous earlier conflicts.

What Jelliman and colleagues suggest is that this defensive function could sometimes be deliberately combined with ecological restoration. Rewetting peatlands or restoring floodplains near vulnerable borders might simultaneously enhance biodiversity, store carbon, reduce flooding and create terrain that is difficult for armoured vehicles to cross. A win-win for both national defence and this wider concept of national security.

Clearly this is a concept that requires much more testing, and ecological restoration should not be distorted into a military land-management programme. There would also be difficult questions about land ownership, farming and the ecological appropriateness of particular interventions. But that is almost beside the point. The fact that rewilding is now being seriously discussed in a defence journal as potential security infrastructure is itself significant.

It challenges the assumption that spending on defence and spending on nature necessarily compete with one another, though we’ve long known that some areas of the UK than are used by the military are also important wildlife sites, Salisbury Plain being an obvious example, the largest known expanse of unimproved chalk grassland in north-west Europe precisely because it is used for military purposes rather than being converted to agriculture.

Losing nature can make countries poorer and less financially secure

Another recent study extends the argument into the financial system. Matthew Agarwala and colleagues published a paper in Nature Ecology & Evolution examining how losses of ecosystem services might affect the creditworthiness of nations, which is the degree to which lenders and investors judge that a country’s government can reliably meet its debt obligations in full and on time. Their model incorporated scenarios involving the deterioration of three services – wild pollination, marine fisheries and tropical timber – into sovereign credit assessments for 23 countries containing about 5.5 billion people.

The numbers produced by their scenarios are striking. Under partial ecosystem collapse, additional annual sovereign interest payments across the countries studied could reach around US$162 billion. India and China alone could experience tens of billions of dollars in increased annual debt-servicing costs. Some countries could suffer very large reductions in GDP.

These are modelled scenarios rather than predictions, of course, and the ecological assumptions that sit beneath such economic modelling need careful scrutiny. But the basic mechanism is compelling.

Governments depend upon functioning economies to raise taxes, borrow money and respond to crises. If ecological degradation reduces agricultural output, fisheries production and other forms of economic activity, the fiscal position of a country deteriorates. Borrowing becomes more expensive precisely when governments may need to spend more money adapting to environmental change.

This summer’s record breaking drought and wildfires in the UK, and the promise of further disruption due to a mega El Nino event, make such adaptation all the more urgent. Nature loss can create a nasty feedback loop: ecological degradation weakens economies, weaker economies have less capacity to invest in resilience and restoration, and that in turn increases their vulnerability to further ecological degradation.

All of this moves biodiversity loss well beyond the conventional environmental policy box and there are positive signs that these ideas are becoming embedded in government.

The UK security machinery is beginning to respond

In June the UK Government established its first Climate Security Taskforce, bringing together experts from the security, military, academic and environmental communities. Significantly, its remit explicitly encompasses not only climate change but nature loss. This is important as many of us have been arguing for years that you cannot disentangle the two and they should not be treated as separate domains of environmental concern. The Government’s announcement stated that climate change and nature loss are drivers of instability, economic disruption and security risk, and linked the Taskforce to the broader approach set out in the UK’s National Security Strategy.

That matters because one of the perennial problems with biodiversity has been institutional fragmentation. Nature tends to be dealt with by environment ministries, while finance ministries think about economic stability, agriculture departments think about food production, health ministries think about disease, and defence and intelligence agencies think about security. But ecological risks do not respect departmental boundaries.

A collapsing ecosystem can simultaneously affect food prices, water availability, infectious disease risks, migration, trade, government finances and geopolitical stability. Treating each of these consequences separately misses the common ecological cause.

China, where I’ve been spending quite a bit of time in recent years, provides an interesting comparison with the UK. Whereas the explicit framing of biodiversity loss as a national-security risk is relatively new in Britain, China has for some years incorporated “ecological security” into its much broader concept of national security. Its first national-security white paper, published in 2025, explicitly listed ecological security alongside military, economic, food, resource, biological and other forms of security. This has been reinforced in 2026 by China’s new Five-Year Plans for ecological protection and the construction of a “Beautiful China”, both of which link biodiversity conservation, ecosystem restoration and resilience to national ecological security. Chinese researchers have meanwhile developed an extensive literature on “ecological security patterns”, identifying the habitats, corridors and ecosystem services required to maintain resilient landscapes. The Chinese use of the term is not identical to the emerging British idea of “nature security”, but the overlap is striking: both ultimately recognise that the security of a state rests partly upon the ecological systems that support it.

From an intelligence assessment to Parliament

The UK Government’s January assessment has continued to reverberate through Westminster. On 2 September, the House of Commons Library published a new briefing ahead of a parliamentary debate on the assessment. The briefing does not constitute a new security assessment, but usefully brings together the original findings with subsequent parliamentary scrutiny, stakeholder responses and government action, including the creation of the Climate Security Taskforce and a new three-year Nature Security R&D Programme.

The briefing rightly emphasises an important point about the original security assessment. It is based on a reasonable worst-case scenario. It is not predicting that these ecosystems will suddenly collapse tomorrow. National security planning routinely explores high-impact possibilities precisely because governments need to understand what would happen if severe events occurred.

On 3 September the subject was then debated in Westminster Hall, following a cross-party initiative led by Adrian Ramsay MP. Whatever ultimately comes from that debate, this represents an interesting political transition. In January, biodiversity loss appeared in a national security assessment, and eight months later it had become the subject of a dedicated parliamentary research briefing and debate. That does not mean that nature has suddenly moved to the centre of British security policy. Far from it. But it suggests that the language of nature security is beginning to acquire institutional traction.

And then there is food

As if to underline the point, today (4 September) the National Audit Office has published a report on the Resilience of the food supply chain to disruptions. This is not primarily a biodiversity report. It examines the resilience of the UK food system to a much wider range of threats, including extreme weather, energy disruption, cyber-attacks, pandemics and animal and plant diseases. But there is a direct connection with the nature-security debate.

Food is one of the UK’s 13 designated Critical National Infrastructure sectors. The NAO concludes that although the food system has proved resilient to previous disruptions, the ability of the sector to withstand catastrophic events has not been tested and that Defra’s actions have not yet been sufficient to ensure resilience to such events.

This brings us back to where I started in January with pollination. Food security is not simply about having enough farms. It depends on soils, water, climatic stability, pollinators, pest regulation, genetic diversity, functioning supply chains, energy, transport and international trade. Pull at enough of those threads simultaneously and resilience begins to unravel.

So where does this leave us?

What interests me most about these developments is that they come from very different intellectual and institutional directions. Ecologists are describing ecosystems as natural infrastructure. Economists are beginning to incorporate biodiversity into sovereign financial risk. Defence researchers are thinking about restored landscapes as strategic assets. Government has created a taskforce dealing with climate and nature security. Parliament is discussing ecosystem collapse as a national security problem. And the National Audit Office is warning that one of the country’s most fundamental pieces of critical infrastructure, its food system, needs greater resilience.

These are not separate conversations, they are pieces of the same emerging picture.

There is, of course, a danger in pushing the national-security framing too far. Nature deserves protection for many reasons that have nothing to do with its usefulness to states, economies or human societies. I would be very uncomfortable with biodiversity conservation being justified solely because it makes Britain, or any other country, more secure.

But that is not the argument I am making. Rather, I think we have systematically underestimated the extent to which national security is built upon ecological stability. Forests, soils, rivers, wetlands, oceans, pollinators and the millions of other species that make ecosystems function are not scenery surrounding the human economy, they are part of its physical foundations.

Earlier this year I argued that conserving pollinators could be regarded as a form of preventive security investment. The developments since then suggest that the same argument can be made much more broadly: Protecting and restoring nature is not an alternative to investing in national resilience. It is one of the ways in which we invest in national resilience.

That feels like an idea whose time has arrived.

There is, however, an obvious limitation to framing all of this in purely national terms. Modern states are embedded in a globalised economy in which food, energy, raw materials, finance, manufactured goods and ecological impacts cross borders continuously. A country may strengthen the resilience of its own landscapes and infrastructure yet remain highly vulnerable to ecosystem degradation, crop failures or political instability elsewhere. In that sense, “national resilience” is also dependent on international ecological resilience: security at home increasingly rests on the stability of environmental and economic systems far beyond national borders. Just as individual trees in a forest are dependent upon one another to create the conditions in which all can thrive, regardless of species, so the too are countries mutually dependent. The leaders of the world’s nations would do well to remember that.

Bird pollination finally confirmed in Britain!

In my book Birds & Flowers, I included a chapter called “The curious case of Europe”. The point of that chapter was simple enough: compared with much of the rest of the world, Europe appears to be oddly deficient in bird pollination. There are no hummingbirds, no sunbirds, no honeyeaters, and very few native plants that obviously look as though they have evolved with birds as their main pollinators. And it Britain, it appears that bird pollination is totally absent.

But “appears” is doing a lot of work there.

For decades, European bird–flower interactions have tended to be treated as marginal curiosities: Blue Tits taking nectar from willow catkins, warblers dusted with pollen, finches messing about in blossom. Interesting natural history, certainly, but not necessarily pollination. The assumption has usually been that insects do the serious work, and birds are at best incidental visitors.

A new paper in Journal of Ecology called “Generalist passerine birds perform a functional role as pollinators in temperate Europe“, by Sandra Anderson, George Perry and Rose Thorogood challenges that assumption in a very useful way. Working at Wicken Fen in Cambridgeshire, they found that pollen transport by passerine birds was widespread. Most of the birds they sampled carried pollen, and several species — including Blue Tit, Blackcap, Chiffchaff, Wren, Redpoll and Bullfinch — regularly carried meaningful loads.

More importantly, they tested whether this mattered to the plants. By excluding birds from flowers while allowing insects access, they showed that fruit-set was reduced in several early-flowering woody plants, including Blackthorn (Prunus spinosa), Hawthorn (Crataegus monogyna) and Buckthorn (Rhamnus cathartica). In other words, the birds were not just getting dusty faces. They were contributing to plant reproduction.

I should say that I was one of the reviewers of this paper, so I have followed its development with particular interest. What I like about it is that it does not try to claim that Europe secretly has a hidden flora of classic “bird flowers”. These are not red tubular blossoms adapted to hummingbirds or sunbirds. They are familiar, open, pale, spring-flowering shrubs and trees. Nor are the birds specialised nectar-feeders. They are generalist passerines making use of seasonal resources.

That is precisely why the paper is interesting. It shifts the question from “does this look like bird pollination?” to “does bird visitation actually function as pollination?” That distinction matters. Pollination syndromes can be useful, but they can also blind us to interactions that do not fit the textbook categories.

The seasonal context is also important. These interactions peak early in spring, when willows, blackthorn and other woody plants are flowering, temperatures are still cool, insects may be unreliable, and birds are preparing to breed or arriving from migration. Under those conditions, even occasional bird visits could be valuable to plants needing pollen moved between individuals.

For me, this paper strengthens the argument I made in “The curious case of Europe”: Europe is not devoid of bird–flower interactions; rather, we have been looking for the wrong kind of bird pollination. Instead of obvious “ornithophilous” specialisation, we may have overlooked a more diffuse, opportunistic, generalist system involving common birds and common spring-flowering woody plants.

That may not be as spectacular as a hummingbird hovering at a tropical flower, but ecologically it is just as revealing.

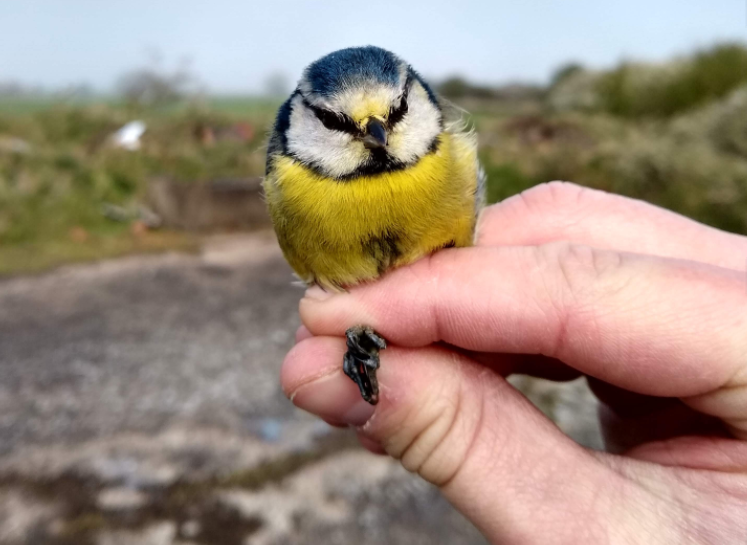
The photo above is from Birds & Flowers and shows pollen on the face of a Eurasian Blue Tit in the early spring. Bird mist-netted under licence in Northamptonshire, UK. (© Lynne Barnett)

Press release: Europe risks a crisis if it fails to halt pollinator loss, researchers warn

NOTE FROM JEFF: This press release came out at the start of the week and I am involved in two of the EU-funded projects that are mentioned, Butterfly and ProPollSoil, and I’m a co-author of the White Paper.

For immediate release

University of Bergen Brussels office, Rue Guimard 1040, Brussels, Belgium, 22 June 2026

Eight EU-funded research consortia warn that Europe risks a crisis if it fails to halt pollinator loss. Their solution: a roadmap to reverse wild pollinator decline and protect managed bees.

A new White Paper from eight major EU-funded pollinator projects warns that the resilience of Europe’s vital societal functions and food security are at stake if the EU fails to halt and reverse wild pollinator declines, and to support managed pollinators. Behind the report is an interdisciplinary team of 135 leading researchers with expertise ranging from ecosystem ecology, pollinator ecology, ecological economics, social science, environmental history, behavioural psychology, political science, and environmental law. The report flags the EU’s siloed governance structures and resulting policy incoherence as the major barrier to pollinator restoration. It states that the EU and its Member States urgently need to act by making Pollinator Stewardship an explicit and measurable top-priority across policies on agriculture, environment, chemicals, research and innovation, trade, finance, planning, legislation, and education.

The report diagnoses the looming pollinator crisis as arising from a dysfunctional relationship between humans and nature. Seeing humans as separate from and superior to nature, and thinking of nature as an object for human use as a resource, reinforces institutional structures that exploit nature for short-term individual and material gain. This leads to unsustainable agricultural practices that risk jeopardising the resilience of the ecosystems on which humanity critically depends.

There is more at stake than food security, the report warns. Indeed, many of Europe’s economic supply chains and sectors depend on pollination of flowering plants. Think of medicinal plants, food supplements, biomass energy crops, biomaterials, textiles, fodder, cosmetics, decoration, art, culture, and tourism.

The report also highlights the low pollinator literacy of key societal actors whose daily actions can make the difference for pollinators. It advocates mandating ecoliteracy in the education of professionals in all key sectors that affect pollinators and their habitats.

According to the report’s lead author, Professor Jeroen van der Sluijs, many people whose actions affect pollinators and their habitat are already doing their best to help save the bees. But most lack the literacy to understand how their practices cascade into pollinator loss.

“Many farmers plant wildflower strips along their fields, but almost no one knows that some moths are more effective pollinators than honeybees. These little creatures of the night, clothed in velvet and moonlit dust, need host plants for their larvae, not only flowers. Host plants for pollinating hoverflies, beetles and moths are missing in most seed-mixtures for flower strips.”

Avoiding a scenario in which Europe is hit by a pollination crisis requires addressing the EU’s functioning and moving away from its siloed governance structures. This requires addressing fragmented responsibilities across sectors, top-down policy design, and weak coordination among administrations that currently hinders effective pollinator restoration. According to the authors, the conflict between short-term production goals and the need to maintain pollination services as a public good must be solved as soon as possible.

The report ends with a detailed roadmap of 15 urgent, evidence-informed recommendations for action that, when fully implemented, can reverse pollinator decline in Europe.

Full White Paper: https://zenodo.org/records/20715669

When an old experiment revealed a new story about flowers

Sometimes, science does not go the way you plan.

That is usually framed as failure: the experiment did not work, the results were inconclusive, the story was unclear. But science can also advance when we go back to old data and ask a different question. That is exactly what happened with a study of Field Scabious, Knautia arvensis, a familiar wildflower of meadows and grasslands.

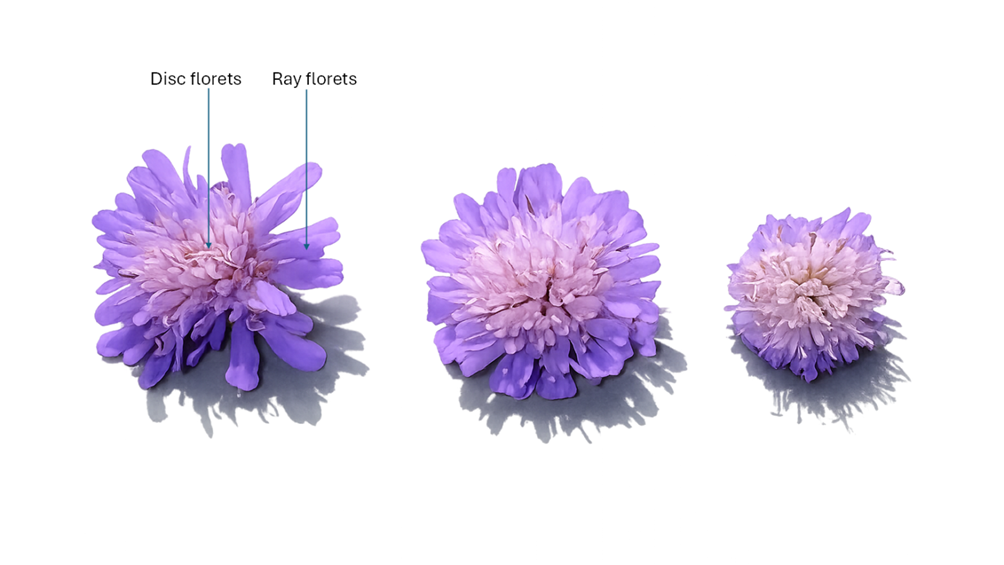
Back in 2001, I carried out an experiment to test the function of the showy outer florets around the edge of the flower head. These enlarged “ray florets” look as though they ought to be important in attracting pollinators. The idea was simple: trim them in different ways and see whether pollinating insects responded – you can see the results of that trimming in the photo above.

The answer, at the time, was baffling. Bumblebees, hoverflies and butterflies (all of which are effective pollinators of this plant) did not seem to care very much. Visitation rates by the insects hardly changed, and neither did seed set. But seed weight did change, as did the amount of sugar being produced by the trimmed flower heads. At the time I could not make sense of this in relation to the question I had asked, so the data were archived and left alone.

But not forgotten.

Fast forward 25 years, and I was chatting about this data set with colleagues when I was at the Kunming Institute of Botany in China. That got me reading some more recent work about florivory -the damage done to flowers by animals – and I realised that this old experiment might make more sense if viewed from another angle. Perhaps I had not really been testing floral attraction at all. Perhaps, without intending to, I had carried out a simulated florivory experiment.

Seen in that light, the results became much more interesting.

Cutting the ray florets did not stop pollinators from visiting. Nor did it reduce the number of seeds produced. But it did change the plant’s internal economics. Nectar quality declined in the most heavily cut flowers, and the seeds that those flower heads produced were consistently lighter. In other words, the flowers still functioned well enough to get pollinated, but the plant appeared to invest less in rewards for pollinators and less in each of its offspring.

That matters because lighter seeds may have poorer prospects later in life, even if the plant initially appears to reproduce successfully. The damage did not cause total reproductive failure. Instead, it produced a subtler effect: hidden costs that only become visible when you look beyond simple seed counts.

Newly contexualised in this way, we wrote up this work, being completely honest about the history of the study, submitted it to the Journal of Pollination Ecology, where it received very positive reviews. It’s now been published and you can download a copy by following the link in the reference:

Ollerton, J., Xu, X. & Ren, Z.-X. (2026) Misconceived experiments may yield valuable insights: simulated florivory has unpredictable consequences for plant reproduction in Knautia arvensis (Caprifoliaceae). Journal of Pollination Ecology (in press)

I like this study because it tells two stories at once. One is ecological: florivory may not always reduce pollinator visits, but it can still alter plant reproduction in potentially important ways. The other is about how science actually works. Not every good paper begins with a perfect hypothesis and a clean result. Sometimes the value lies in returning to an awkward, neglected dataset and realising that it was trying to tell you something different all along.

Science does not always go the way you plan. But occasionally that is when it becomes most revealing.

What the COVID lockdowns taught us about plant-pollinator specialisation in gardens

One of the few positive things to come out of the COVID lockdowns was the unexpected opportunity to look much more closely at the nature right outside our doors. In 2020 I coordinated the Lockdown Gardens initiative, bringing together pollination ecologists from around the world to carry out standardised surveys of flower visitors in the gardens they could access during that strange and constrained period. That project generated an unusually rich global dataset: 67 gardens, almost 47,000 flower visits, and records from more than 650 pollinator species.

Since then, the dataset has started to yield some really interesting insights. A new paper led by Luis Perugini uses the Lockdown Gardens data to ask a deceptively simple question: what determines how specialised plant–pollinator interactions are in gardens? In other words, are garden flowers in some places visited by a narrow set of pollinators, while elsewhere they are more generalist?

The answers are not quite what we expected. Looking at 40 garden networks from four continents, we found that larger gardens support more plant species, and that suburban gardens tended to be richer in plant species than either rural or urban gardens. We also found that pollinator richness increased with plant richness and with precipitation. But when it came to the actual specialisation of interactions, climate and species richness did not seem to matter very much at all. Instead, variation in specialisation was mostly species-specific and showed no clear phylogenetic pattern.

That’s an important result, because it suggests that the factors that drive biodiversity in gardens are not necessarily the same factors that shape the ecological relationships within those gardens. Put more simply: having more species does not automatically mean having more specialised interactions.

For me, this is a nice example of how a project born out of a global crisis can continue to produce useful science. The Lockdown Gardens surveys began as an improvised response to an extraordinary moment, but the data are now helping us to understand how gardens function as ecological systems, and how they might better support pollinators in an increasingly human-dominated world.

Here’s the full reference with a link to the paper, which is open access:

Perugini, L., Rech, A., Ollerton, J. & Jorge, L. (2026) Global drivers of plant-pollinator interaction specialization in gardens. Ecology and Evolution (in press)

Edible Apocynaceae: a new global synthesis of diversity, conservation and pollination just published – and a personal landmark for me!

This year – 2026 – marks the 40th anniversary of my first publication. Forty years. Imagine that – I certainly can’t! It feels like a long time ago, a distant memory, another life. I was 21 and I hadn’t even begun my undergraduate degree. After a less-than-successful time at school I decided to complete a Higher National Diploma (HND) qualification in Applied Biology at Sunderland Polytechnic (now the University of Sunderland) that I hoped would get me a place on a degree course. As it turned out, it did, but during my HND I completed a research project which (with the encouragement of my then supervisor, the late cactus expert Geoff Swales*), was subsequently published in December 1986 as “Adaptation to arid environments in the Asclepiadaceae” in the British Cactus and Succulent Journal.

That was the modest start of a botanical love affair with asclepiads (now subsumed into the family Apocynaceae) that has persisted to this day and resulted in over 20 research papers, chapters, and more general articles, plus appearances in both of my books.

The latest of these papers is published today and, as well as being a 40 year milestone for me, it’s a paper that I am inordinately proud of, as it represents an amazing coalescence of ethnobotany, taxonomy, conservation, biogeography, cultural science, and pollination ecology. And I managed to sneak in a citation of the 1986 paper that started the whole thing!

This paper is the first global review of the diversity of edible species in a family that is usually considered to be highly toxic and produces a lot of sticky latex to deter herbivores. Yet that reputation turns out to be only part of the story. Our survey found no fewer than 440 edible species of Apocynaceae worldwide, which works out at about 7.7% of the family (and is definitely an under-estimate). They occur across all of the major evolutionary lineages of the family, and in most of the main biogeographic regions where these plants grow.

What people eat is also far more varied than you might expect. Fruits are the commonest edible part, but roots and tubers are also important, and in different places people consume leaves, stems, flowers, nectar, latex, bark and even wood ash used as a condiment. That diversity is not random: our analyses show clear phylogenetic and geographic patterning in which parts are eaten. In other words, both evolutionary history and regional cultural practices help to shape how Apocynaceae are used as food.

One especially interesting result is that edible Apocynaceae appear, on current evidence, to be less threatened than non-edible members of the family. But that comes with a big health warning: more than 80% of species, edible or otherwise, have never been properly assessed for conservation status. So there is still a huge amount that we do not know.

The same is true for pollination. Many of these plants depend on animal pollinators to produce the fruits and seeds that people eat, yet pollination data are missing for most edible species, including about 90% of those whose edible parts are directly pollinator-dependent.

For me, that is one of the most striking messages of the paper. Hidden inside a family best known for poisons and medicinal compounds is a substantial, globally distributed food resource, much of it tied to local knowledge and wild harvesting. It is a reminder that botanical and cultural diversity, conservation, and pollination ecology are all bound up together. And, as a nice bonus, the study even uncovered an unexpected taxonomic surprise in China, where one edible species turned out to belong in an entirely new genus, Kushengia. The edible flowers of Kushengia sinensis are shown in the image at the top of this post – lightly boiled, stir fried with garlic, and thoroughly delicious!

Here’s the reference with a link to the paper, which is unfortunately pay-walled. If anyone wants a copy, send me a request via my Contact page:

Ollerton, J., Albuquerque-Lima, S., Liede-Schumann, S., Galetto, L., Endress, M.E., Forster, P.I., Torres, C., Fishbein, M. & Ren, Z.X. (2026) Edible Apocynaceae: phylogeny, biogeography, conservation and pollination insights from a global synthesis. Taxon 75: e70131

*It goes without saying that I’m incredibly grateful to Geoff and the other teachers and supervisors who, during the course of my education, encouraged me in my studies. During one lab session with Geoff we were each given a cactus seed and asked to study it under a microscope and draw it. Afterwards I pocketed the seed, took it home, and germinated it. That cactus – a specimen of Parodia (Notocactus) mammulosus – is still growing on my windowsill, a living reminder of a great mentor.