
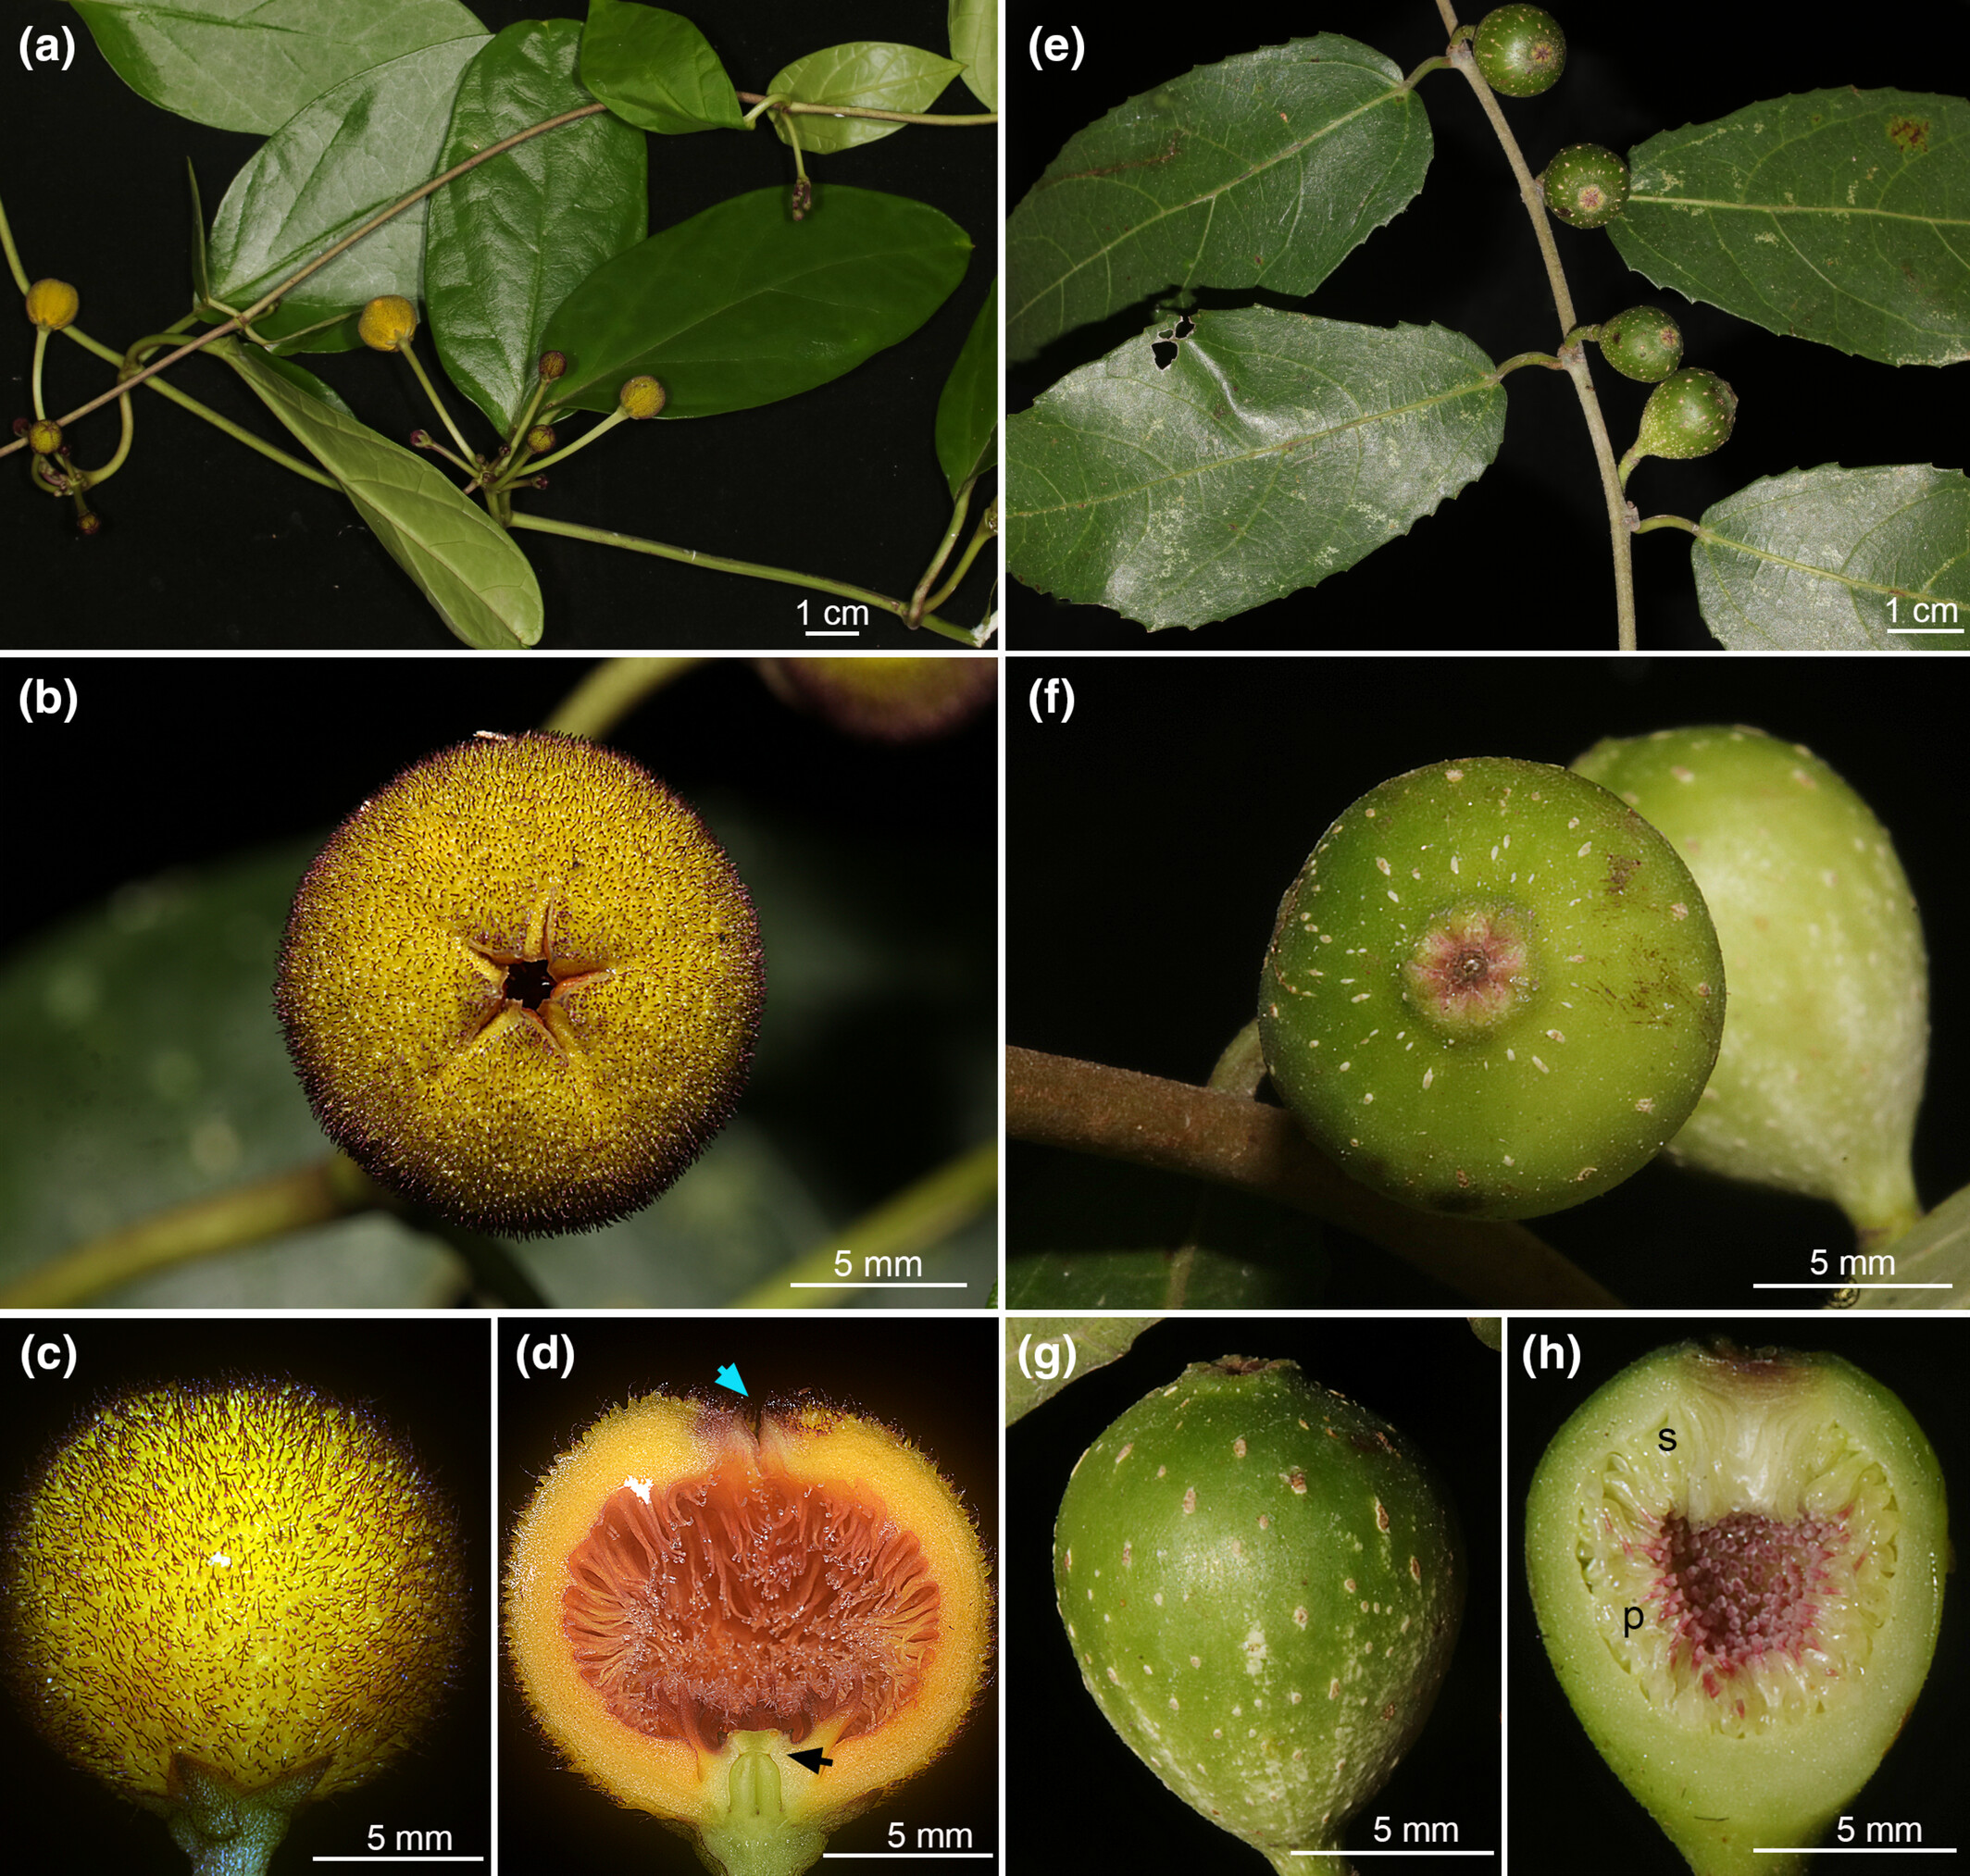
One of the things I love about working on the milkweed and dogbane family (Apocynaceae) is that it has an apparently inexhaustible capacity to produce strange and wonderful interactions with animals. Just when you think that the family’s pollination biology has yielded most of its surprises, along comes something like this.
A paper just out in New Phytologist, led by Aroonrat Kidyoo, describes the pollination of Heterostemma ficoides, an unusual climbing plant from northern Thailand. The title rather neatly gives away the story: “Fake figs, fooled fig wasps and rewarded phorid flies: brood-site mimicry and mutualism in Heterostemma ficoides (Apocynaceae)”.
And “fake figs” is not journalistic exaggeration, as you can see from the photos above, which are taken from the paper. The flowers of H. ficoides are globose, fleshy structures, about 1.5–2 cm across, with a small opening at the top. Superficially they look remarkably like the enclosed inflorescences (the syconia) that we normally call figs. Indeed, when the species was first described in 2019, its resemblance to a fig was obvious enough to inspire the name ficoides: fig-like. But looking like a fig is only the beginning of the story.
Fooling one of nature’s most specialised pollinators
The relationship between figs (Ficus) and their tiny agaonid wasps is one of the classic examples of an intimate plant–pollinator mutualism. Female fig wasps locate receptive figs using their scent, squeeze through the tiny opening or ostiole, and pollinate the enclosed flowers while attempting to reproduce inside. These relationships can be remarkably specific, in some cases representing rare examples of one-to-one plant-pollinator interactions.
So it was genuinely surprising to discover female Kradibia fig wasps entering flowers of Heterostemma ficoides. These wasps normally pollinate Ficus heterophylla, not an Apocynaceae, and the authors believe that nothing comparable, i.e., a fig wasp being fooled into visiting a completely unrelated flowering plant, has previously been documented. I have to concur, this relationship is (so far) unique.
The authors have neatly demonstrated that the deception of these wasps is not simply visual. The chemical bouquet produced by H. ficoides is closer to that of receptive Ficus heterophylla figs than it is to the flowers of its relative H. siamicum. More importantly, behavioural experiments showed that Kradibia wasps were significantly attracted to the scent of open H. ficoides flowers, though not to unopened flower buds. In other words, the plant seems to switch on its misleading olfactory advertisement at just the right time.
Once inside, however, the wasps discover that they have made a serious mistake. They wander around probing the inner surface, searching for egg-laying opportunities that simply aren’t there. Some die inside the flower, although more than 80% of observed individuals managed to get out again, and often went on to visit another Heterostemma flower.
In the process, pollen can be transferred between flowers, but as in other members of the Asclepiadoideae, Heterostemma does not dust its visitors with loose pollen grains. Instead, pollen is packaged into pollinia which become attached to the legs of the fig wasps.
So from the fig wasp’s perspective this is straightforward deception: the plant promises a breeding site that doesn’t exist, and the flowers get pollinated in return. But that is only half of the system.
The flies are not being fooled by the fake fig
The most important pollinator of H. ficoides appears to be a tiny phorid fly in the genus Megaselia, and its relationship with the plant is quite different. Female Megaselia enter the flowers and lay their eggs there. Mating may even take place on the flower beforehand. Their larvae then develop inside the fallen flowers, eventually completing their development in the decomposing floral tissue on the forest floor. For these flies the promise made by the flower is therefore an honest one: this really is a brood site.
Pollinaria become attached to the flies’ mouthparts, then the flies carry them to another flower, where pollen can be deposited. Interestingly, Megaselia are also important pollinators of some species of the related Ceropegia in Africa (both genera are members of the tribe Ceropegieae).
This creates an ecological combination that is one of the most distinct examples of a “bimodal pollination system” that I’m aware of, in which the same flower operates simultaneously as a brood-site mutualism and as a brood-site deception, involving two completely distinct groups of insects.
Back to our 2019 Apocynaceae review
For me, there is a satisfying connection here with the large review of Apocynaceae pollination systems that we published in Annals of Botany in 2019: The diversity and evolution of pollination systems in large plant clades: Apocynaceae as a case study. Aroonrat Kidyoo, lead author of this new study, was also one of the large international team involved in that paper.
We assembled usable pollination information for 567 species (a bit more than 10% of the family) and found an extraordinary diversity of interactions. About 73% of the species for which we had information were associated predominantly with a single broad pollinator group, whether bees and wasps, butterflies and moths, flies, beetles or birds. However, about 7% of the species had distinct bimodal pollination systems, such as bee + butterfly. Whether this is an unusually high proportion for such a family is currently unclear as there are few comparative statistics.
One of our broader conclusions from the study was that this interaction diversity was not randomly scattered across the Apocynaceae evolutionary tree. Pollination systems show strong phylogenetic structure and some transitions between pollinator types have occurred much more readily than others. The new Heterostemma study puts some wonderfully detailed natural history onto that much larger evolutionary picture.
Aroonrat and her colleagues suggest that Heterostemma ficoides may represent a shift away from the more open, nectar-producing flowers found in other parts of the genus. In section Oianthus, to which H. ficoides belongs, the flowers have become progressively more closed. In the extreme case represented here, the result is a globose chamber entered through a small opening, nectar production has apparently disappeared, and the plant has moved towards brood-site pollination by flies and deception of fig wasps.
Whether that evolutionary scenario survives a proper phylogeny and detailed pollination studies of the remaining species is an obvious question for the future. As the authors themselves acknowledge, both are currently lacking. But it is exactly the sort of transition that our 2019 study suggested we should be looking for.
And what does any of this have to do with eating Apocynaceae?
Quite a lot, in a roundabout way. Earlier this year my colleagues and I published another large synthesis of the family, this time asking a very different question: which Apocynaceae do people eat?
We documented 440 edible species, spread widely across the evolutionary tree of the family. That sounds like a lot, although statistically Apocynaceae are actually under-represented among the world’s food plants, probably in part because the family is so well endowed with toxic and pharmacologically active chemistry.
One point that emerged strongly from that work was that our knowledge of how those useful plants reproduce is remarkably incomplete. Many edible Apocynaceae are harvested for their fruits and seeds, which of course ultimately means that successful reproduction matters. Yet for most of those species we still know little or nothing about their pollinators.
That matters if we are serious about conserving wild food plants or developing some of them as future crops. You cannot fully understand the biology of a fruit-producing plant without understanding how the flowers get pollinated in the first place.
There are no Heterostemma species documented in our edible-plant study, so H. ficoides is not some promising new food species. But that isn’t my point. Rather, this new research is a reminder of just how much biological complexity can lie behind the production of an Apocynaceae seed. And we still know the pollination biology of only a fraction of this enormous family.
That, perhaps, is the broader lesson from all three papers. Large databases and family-wide syntheses are valuable because they reveal general patterns and, equally importantly, the gaps in our knowledge. But filling those gaps still depends on researchers spending time watching individual plants and individual insects, dissecting flowers, rearing larvae and asking exactly what the animals are doing. Sometimes what they find is stranger than anyone would have predicted.



 Prof. Jeff Ollerton - ecological scientist and author
