Category Archives: Pollination

Insects do far more than pollinate: a new review of their contributions to people

When we talk about the importance of insects to human societies, the conversation often turns quickly to pollination, particularly the role of bees and other insects in producing the food that we eat. As someone who has spent much of his career studying pollination, I’m probably partly responsible for that emphasis!

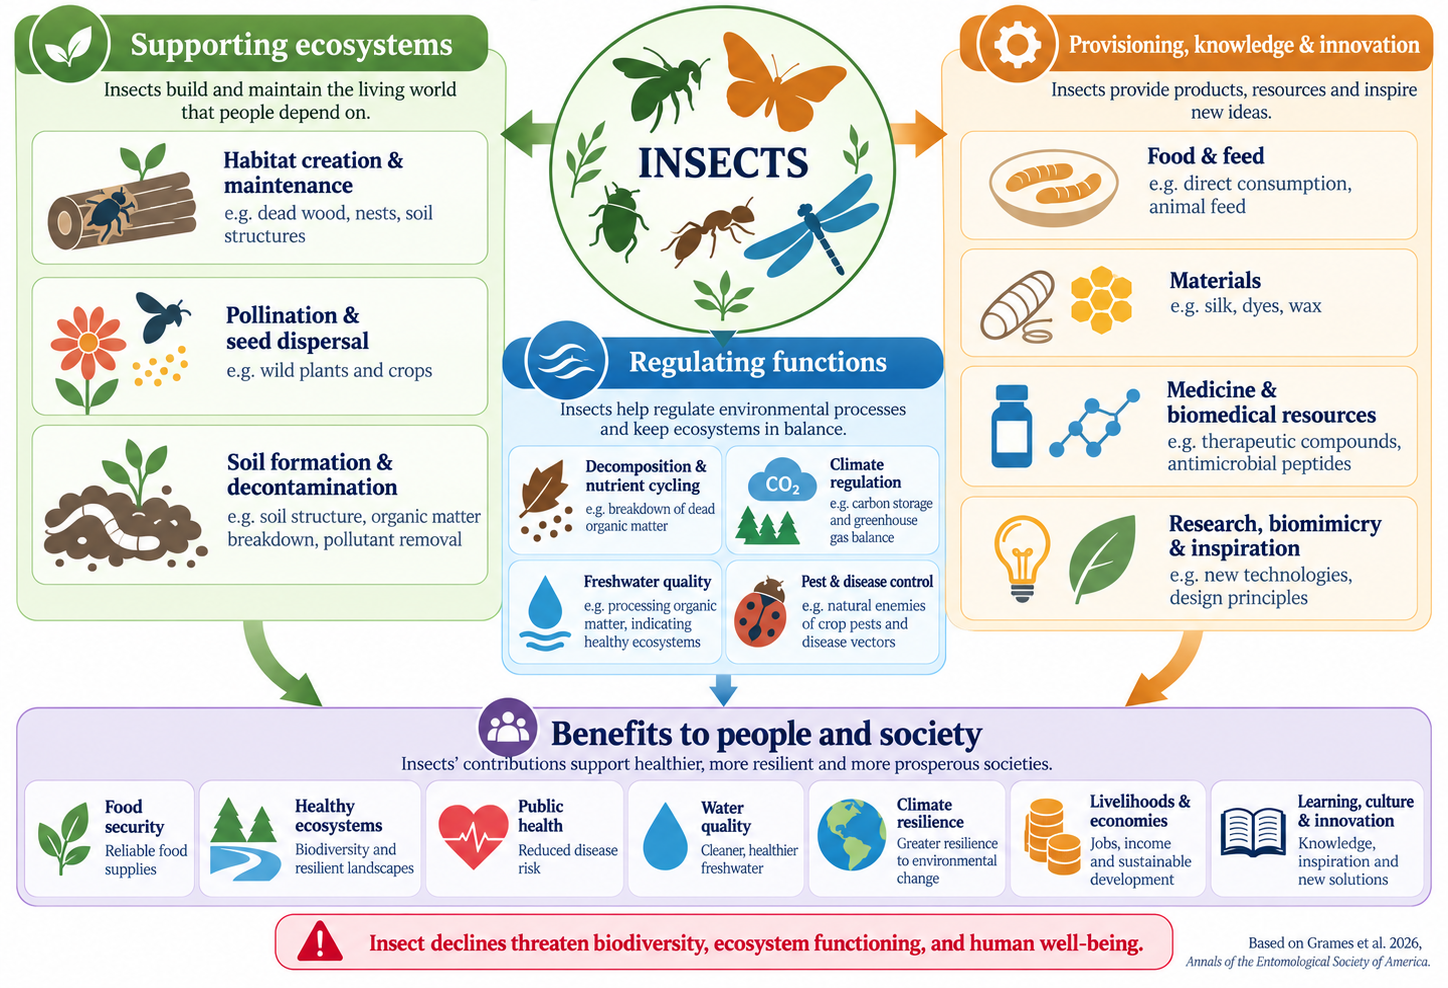
But insects do an enormous amount more than move pollen between flowers. A new review that I’ve co-authored with Eliza Grames and a large international group of colleagues, published in the Annals of the Entomological Society of America, explores the extraordinary range of ecosystem functions and services that insects provide.

And some of these are rather surprising. Of course, pollination is an important part of the story. An estimated 80–90% of flowering plants depend on animals for pollination, overwhelmingly insects. But consider some of the other contributions that our review brings together:

  • Dung beetles remove animal faeces, recycle nutrients, improve soil structure and reduce the abundance of livestock parasites. One study estimated that their activities could be worth around £367 million annually to the British livestock industry.
  • Carrion-feeding flies and beetles help dispose of dead animals and recycle their nutrients.
  • Termites and ants are major ecosystem engineers, creating habitats used by numerous other species and influencing the structure of plant communities.
  • Aquatic insects help maintain water quality, transfer nutrients between freshwater and terrestrial ecosystems, and provide food for fishes and other animals.
  • Then there are the more direct contributions to human societies. Insects provide silk, dyes, medicines and materials for industry. The use of fly larvae to clean wounds is a particularly striking example of something that might initially seem rather unpleasant but is medically valuable!

What I particularly like about this review is that we don’t simply catalogue these contributions. We also assess the strength of the scientific evidence supporting them, using the framework developed by the Intergovernmental Science-Policy Platform on Biodiversity and Ecosystem Services (IPBES). Some services, including pollination, decomposition and biological pest control, are very well established. Others, such as the potential for insects to remove environmental contaminants, remain much less understood.

There’s a connection here to our recent review of the importance of insects to vertebrates, which I wrote about last month. Both papers emerged from the international Status of Insects Research Coordination Network, and both emphasise how deeply insects are embedded in the ecological processes that sustain life.

It also connects with something I’ve discussed in relation to plant–pollinator interactions: we need to look beyond the familiar species and interactions if we want to understand how ecosystems really work.

One important message from the new review is that the value of insects cannot be captured simply by attaching monetary figures to the services they provide. Some of their contributions are extraordinarily difficult to quantify, and many are essential to the functioning of ecosystems regardless of whether humans benefit from them directly.

E.O. Wilson famously described insects and other invertebrates as “the little things that run the world”. Almost forty years later, we’re still discovering just how accurate that observation was.

The paper is open access and can be read here:

Grames, E.M., Noriega, J.A., Sanchez Herrera, M. et al. (2026) Insects’ contributions to people: ecosystem services and functions provided by insects. Annals of the Entomological Society of America. https://doi.org/10.1093/aesa/saag038

My thanks to Eliza and all the other colleagues involved in bringing together such a wide-ranging review.

October good news: Birds & Flowers goes Japanese and I am awarded a fellowship!

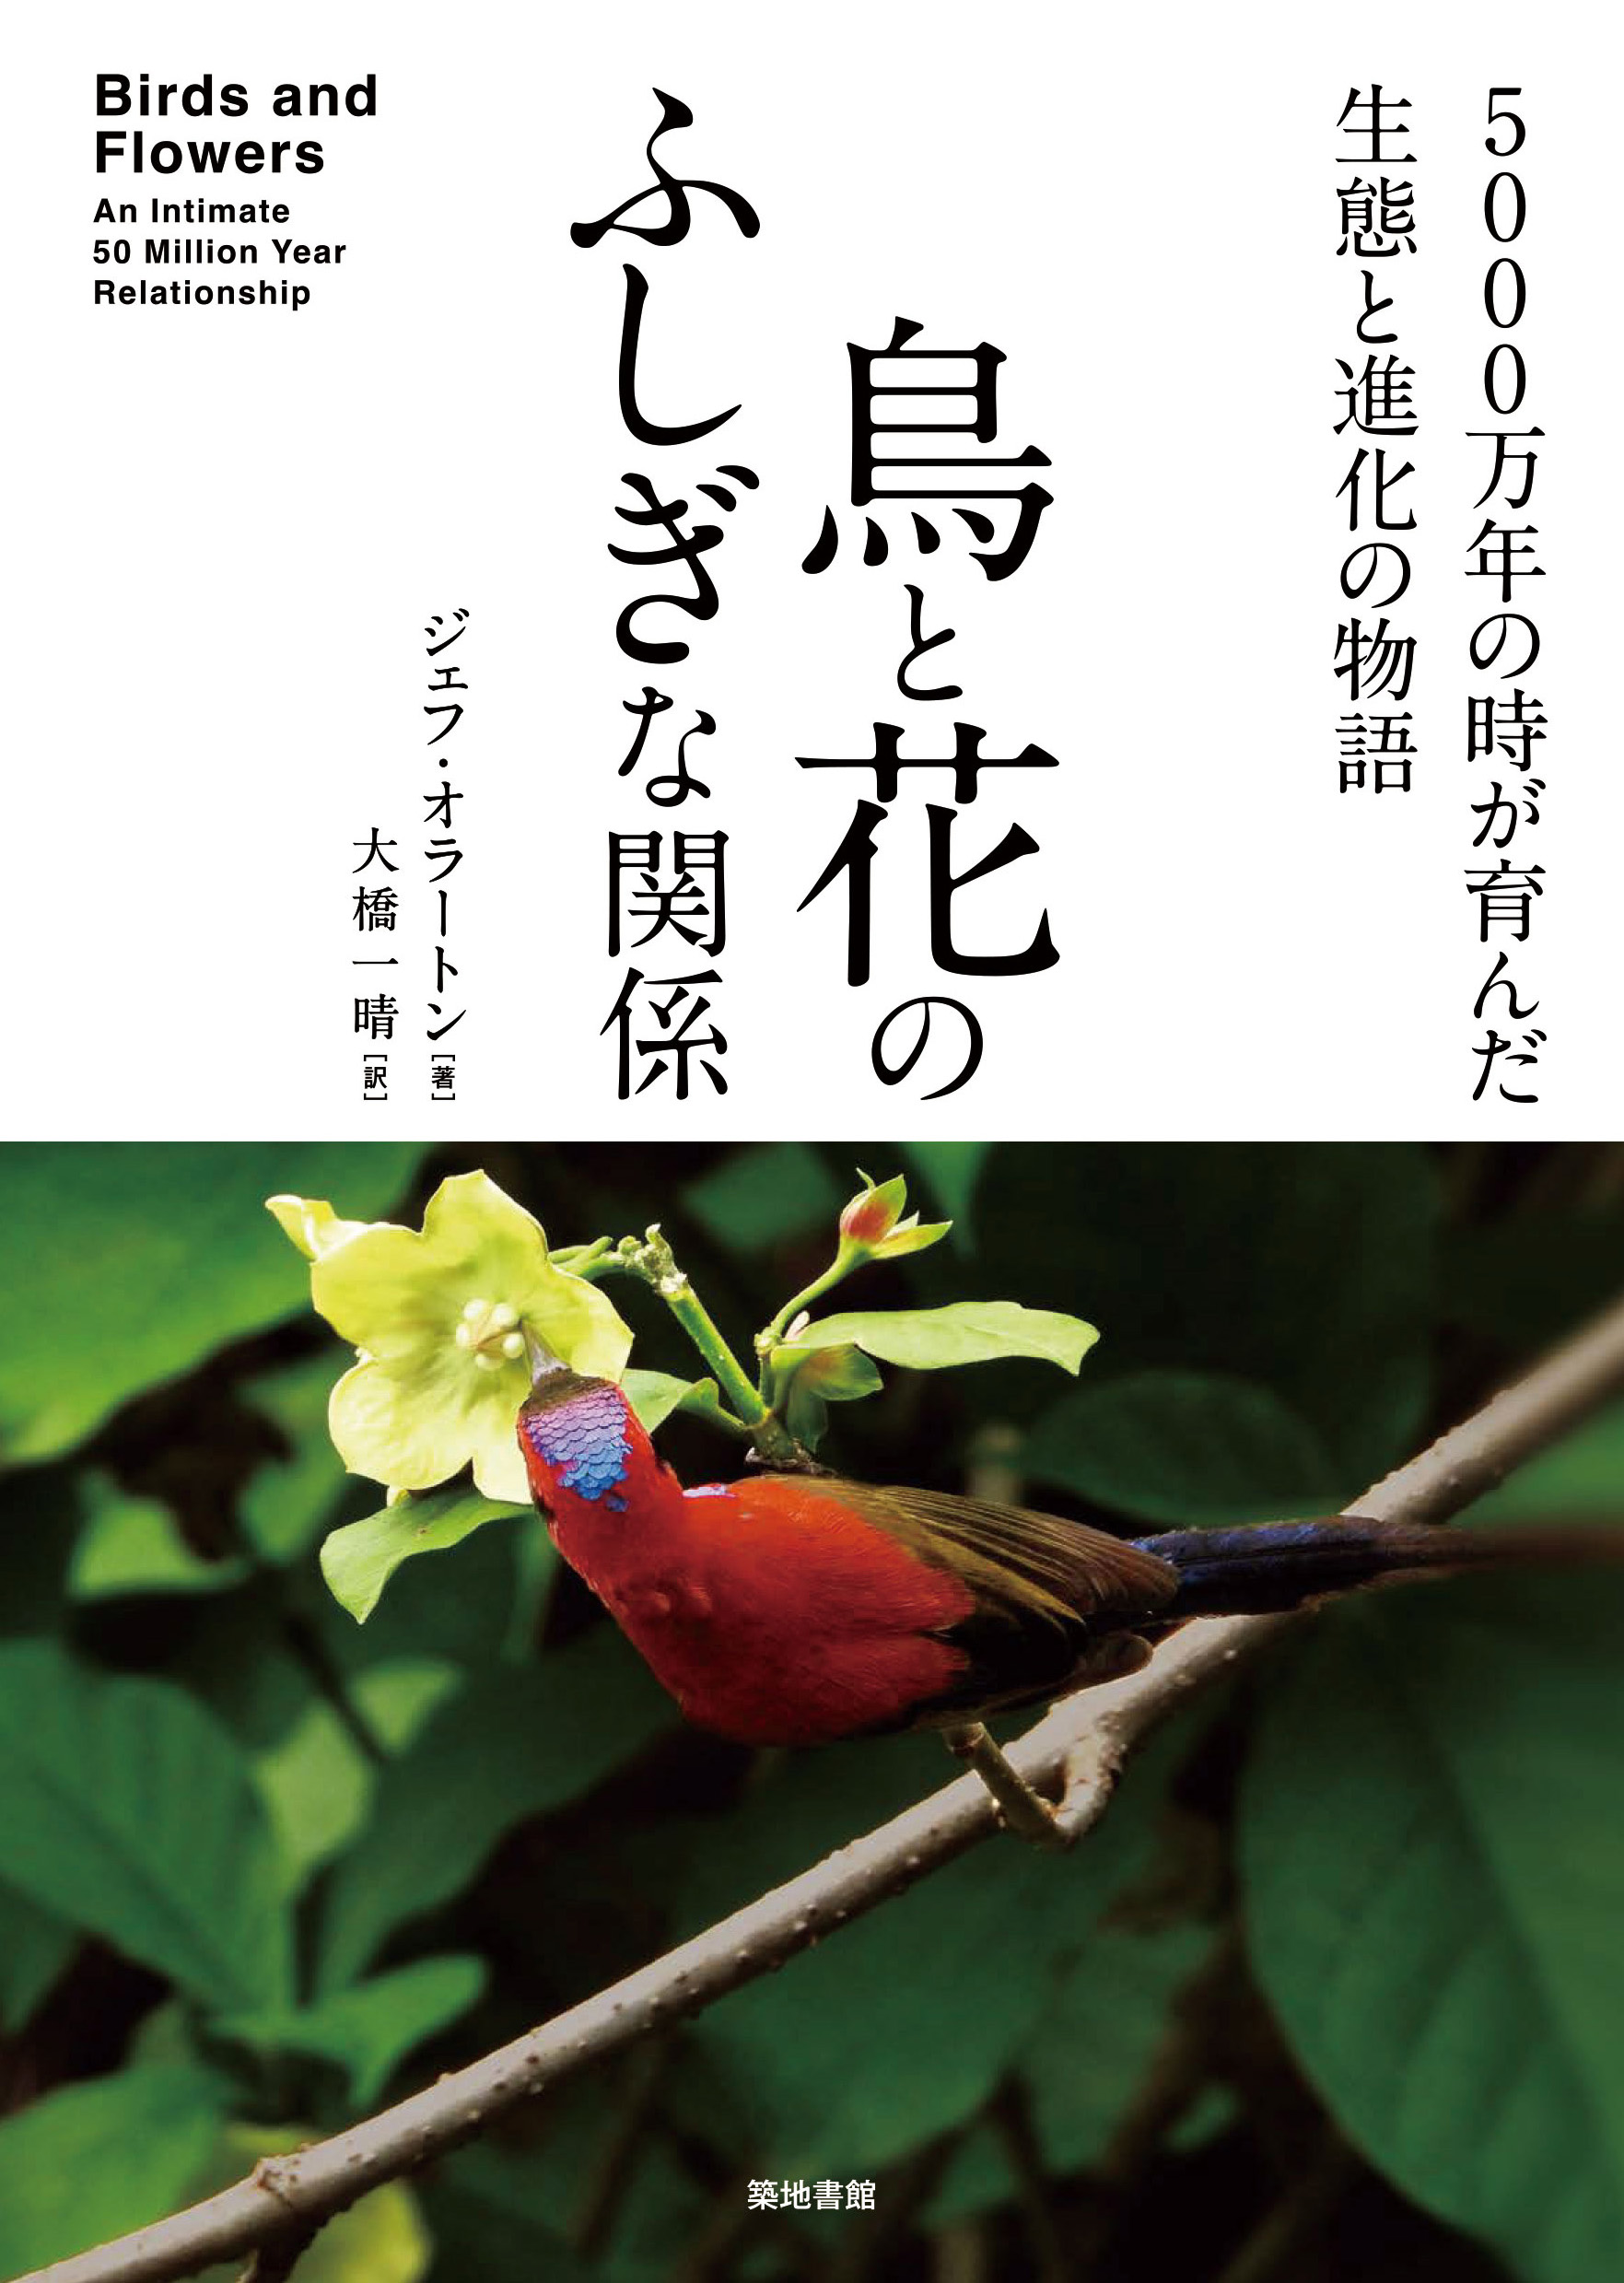
It’s been a good month for me, with two pieces of news that I wanted to share with readers of this blog. First, I’m delighted to announce that my book Birds & Flowers: An Intimate 50 Million Year Relationship has been translated into Japanese! The new edition, published by Tsukiji Shokan, is titled 『鳥と花のふしぎな関係』, which translates roughly as The Curious Relationship Between Birds and Flowers. The subtitle is A Story of Ecology and Evolution Shaped by 50 Million Years. It’s the first foreign-language translation of the book, which was originally published by Pelagic Publishing in February 2024. The Japanese edition is scheduled to go on sale on 18th November.

I’m particularly pleased with the cover, which you can see above. It’s very different from the English edition, with its striking vertical Japanese lettering and a beautiful photograph of a bird (a male Mrs Gould’s Sunbird) visiting a flower (Vallaris indecora – Apocynaceae), taken by my colleague Sinzinando Albuquerque-Lima. There’s something rather special about seeing words that you’ve written transformed into another language, particularly one that you can’t read yourself! My thanks go to the translator, Kazuharu Ōhashi (大橋一晴), and everyone involved at Tsukiji Shokan for bringing the book to a new readership.

One of the things that motivated me to write Birds & Flowers was the realisation that, despite decades of research on bird pollination, nobody had attempted to bring together the full diversity of these interactions in a single book aimed at a broad readership. Hummingbirds are familiar to most people, of course, but bird pollination extends far beyond them, involving an extraordinary diversity of birds and flowering plants across the world.

Japan is an interesting place for this book to appear. Although it lacks the spectacular specialised bird-pollination systems that we associate with tropical regions, East Asia has its own fascinating bird–flower relationships, some of which remain poorly understood. Indeed, as I discussed earlier this year, we’re still discovering just how important birds can be as pollinators even in places where they have traditionally been overlooked, including Britain.

I hope that the Japanese edition will introduce these ecological relationships to a new audience, and perhaps encourage more people to look closely at the interactions between birds and flowers in their own surroundings. You can find details of the Japanese edition on the publisher’s website.

The second piece of good news is that I’ve been awarded a Fellowship of the British Ecological Society (FBES), in recognition of my “significant contribution to ecology and leadership within the ecological community”.

Typically, I’m not a natural joiner of organisations. There’s a raft of societies that I could be a member of and use the post nominals, but but I’m particularly pleased about this award because the British Ecological Society has been an important part of my professional life for many years (I joined in 1990!) It’s the world’s oldest ecological learned society, and its Fellowship recognises contributions across research, teaching, conservation, policy and the wider application of ecological science.

As I wrote earlier this year, 2026 marks the 40th anniversary of my first scientific publication, which appeared in the British Cactus and Succulent Journal in December 1986, when I was just 21. At that point I hadn’t even started my undergraduate degree, and certainly had no idea where my interest in plants, pollination and ecology would eventually take me.

Forty years later I’m still asking questions about how plants and animals interact, still finding things that surprise me, and still enjoying the process of doing science and communicating it to other people. It’s been a career shaped by an enormous number of colleagues, collaborators, students, teachers and friends, many of whom have challenged my ideas, introduced me to new ones, and encouraged me to pursue questions that I might otherwise have overlooked. So I’m very grateful to the BES for this recognition, and to all those people who have been part of the journey.

A Japanese translation and a Fellowship in the same month. Not a bad way to round off the 40th anniversary year of my first publication! And there’s still plenty more science, and writing, to come.

Bees, moths, cockroaches and some unfortunate flies: the surprising pollination of a European milkweed

Back in October 2021, I wrote a post about tracking down a rather elusive plant on the Danish coast. Karin and I had been cycling around the Odsherred region when I spotted the distinctive yellowing autumn foliage of Vincetoxicum hirundinaria growing close to the little fishing harbour at Klint.

I was particularly pleased to find it because Vincetoxicum is a genus of plants that I’ve been interested in for many years. It’s part of the milkweed and dogbane family, Apocynaceae, and belongs to the subfamily Asclepiadoideae, a group with some of the most extraordinarily complex flowers in the plant kingdom.

At the end of that post I asked a question: what was pollinating those flowers on the exposed Danish shoreline? At the time there were surprisingly few published records of pollinators for this widespread European species.

Five years later, I’m delighted to say that a new paper just published in AoB PLANTS, led by my Chinese colleague Wujian Xiong, and to which I’ve contributed, goes a considerable way towards answering that question. Not specifically for the Danish population, but for several populations studied in and around Salzburg, Austria. And the answer is rather more complicated, and interesting, than we might have expected.

A very specialised flower with remarkably unspecialised tastes

The flowers of Vincetoxicum hirundinaria are small, pale cream or ivory-coloured, and about 12 mm across. Like other members of the Asclepiadoideae, they have a highly specialised mechanism for transferring pollen.

Rather than producing individual loose pollen grains, the pollen is packaged into structures called pollinia, which are joined together by a central attachment mechanism to form a pollinarium. When an insect visits a flower, part of its body can become caught in a narrow guiding structure. As it pulls away, a pollinarium may become attached to its mouthparts, legs or other appendages. If all goes well, the insect carries that pollen to another flower and deposits it into a specialised receptive chamber.

It’s an extraordinarily precise mechanism, and one might reasonably expect that only a rather narrow range of insects could operate it successfully.But that’s not what we found.

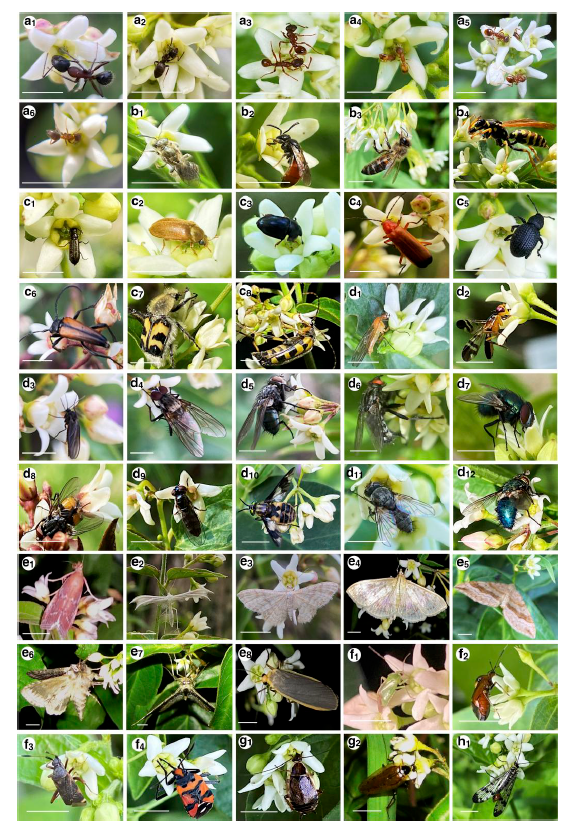
Over 50 hours of observations, Wujian recorded almost 3,000 visits to the flowers, involving 81 species or morphospecies of insects from seven different orders. These included bees, wasps, ants, flies, beetles, moths, bugs, scorpionflies and cockroaches.

Of those 81 types of flower visitor, 37, representing five insect orders, were found carrying pollinaria. These included 15 types of flies, seven bees and wasps, seven moths, six ants, one beetle and one cockroach. That’s a remarkably diverse assemblage for a plant with such specialised floral structures. Indeed, it’s the most diverse pollinator assemblage so far documented for any member of Vincetoxicum.

What makes this particularly interesting is that the pollinaria were attached to different parts of the insects’ bodies. In flies they might be on the proboscis or legs; in bees and wasps on the mouthparts; in moths on the proboscis; and in cockroaches on the labial palps.

In other words, the same elaborate floral mechanism can operate with insects that differ enormously in their anatomy, size and behaviour.

Another chapter in the story of cockroach pollination

There’s a particularly satisfying connection here with another paper that Wujian and I published back in 2020. That study demonstrated specialised cockroach pollination in the rare and endangered Chinese species Vincetoxicum hainanense. Its small flowers open at night, produce an unpleasant scent reminiscent of rotting fruit, and are principally pollinated by a particular species of cockroach, Blattella bisignata.

It was the first documented example of specialised cockroach pollination in the Apocynaceae, and one of only a handful of well-studied examples from anywhere in the world. Now we have another species of Vincetoxicum that is visited and potentially pollinated by cockroaches, but in this case they are just one component of a much more diverse assemblage.

The contrast between the two species is striking. They share the same basic type of highly specialised floral architecture, yet one has a relatively narrow pollination system while the other is much more generalised. Clearly, floral complexity doesn’t necessarily translate into ecological specialisation.

Day and night, and the importance of place

Another interesting finding concerns when the flowers are available to pollinators. The flowers of V. hirundinaria open in the late afternoon, between about 4pm and 6pm, and remain open for an average of six days. They produce nectar and a strong, sweet scent that we describe in the paper as reminiscent of red wine.

That long floral lifespan means that they are potentially accessible to both daytime and nocturnal insects. But the relative importance of those insects varied considerably between the study populations. At most sites, pollen removal and deposition took place during the day, with bees, wasps and other diurnal insects playing the main roles. However, at the higher-elevation Gaisberg site, nocturnal moths and cockroaches were much more prominent, and pollen transfer during the night was particularly effective.

It’s a useful reminder that a plant doesn’t necessarily have one fixed set of pollinators across its geographical range. The animals available to visit flowers can change with location, habitat, season and time of day. This connects with some of the arguments that I’ve made recently about geographical variation in plant–pollinator specialisation. Ecological specialisation isn’t always an intrinsic, unchanging characteristic of a species, it can depend very much on the circumstances in which that species is studied.

But not every visitor is a useful pollinator

There’s a rather darker side to this story, however: the flowers of Vincetoxicum hirundinaria can be surprisingly dangerous places for small insects. We recorded 16 types of flies that became trapped by the flowers, often fatally, when their mouthparts became lodged in the structures associated with the pollinarium. Some were simply too small or weak to pull themselves free.

This phenomenon is known from other milkweeds, including the notorious moth-catching vine Araujia sericifera. However, the extent of insect trapping that we observed in V. hirundinaria was quite remarkable. There’s an important distinction here between attracting an insect to a flower and actually using it to transfer pollen successfully, even for those species that don’t get trapped.

Ants, for example, accounted for about a quarter of all recorded flower visits, but only 3.5% of the sampled ants carried pollinaria. In contrast, between 40% and 60% of individuals in several other insect groups carried pollinaria.

Even carrying a pollinarium doesn’t necessarily mean that an insect will successfully deposit pollen into another flower. That requires the insect to visit a suitable flower and position its body in just the right way. I’ve discussed this issue before in relation to what we actually mean by a pollination system. Counting floral visitors is relatively straightforward. Demonstrating that those visitors contribute to successful plant reproduction is much more difficult.

In the present study, the evidence for functional generalisation is strong in terms of the diverse insect groups capable of removing and transporting pollinaria. However, we cannot yet say precisely how much each group contributes to successful pollen deposition and seed production.

Indeed, overall pollen transfer efficiency was quite low. At most sites only about 3–9% of the pollen removed from flowers was successfully transferred to another flower’s receptive structures during the day. At Gaisberg, nocturnal pollen transfer efficiency averaged around 11%. Nor did the plants produce many fruits. Only 2% of naturally pollinated flowers produced mature fruits, compared with 14% following experimental cross-pollination. The plants were also self-incompatible in the populations we studied, meaning that pollen transferred between flowers of the same individual wouldn’t result in successful reproduction.

So despite attracting a remarkably diverse range of insects, V. hirundinaria appears to have substantial limitations on its reproductive success. Pollination isn’t simply a numbers game.

Back to the bigger picture

Readers of this blog will know that the diversity and evolution of pollination systems in Apocynaceae has been a major theme of my research for many years. In our large international review published in 2019, we brought together information on the pollinators of 567 species and showed that the family encompasses everything from extremely specialised relationships to highly generalised systems involving many different kinds of animals.

More recently, I’ve written about the extraordinary pollination biology of Heterostemma ficoides, which deceives fig wasps while providing genuine breeding opportunities for tiny flies. And only last week I discussed our new study of eleven co-occurring Apocynaceae species in Argentina, showing how very different flowers can share overlapping assemblages of visitors.

The new Vincetoxicum study adds another piece to this evolutionary and ecological puzzle. It demonstrates that even one of the most mechanically sophisticated types of flower can function with a very wide range of potential pollinators. Floral specialisation and pollinator specialisation are not the same thing, and we shouldn’t assume that one necessarily predicts the other.

But it also raises some intriguing questions. Why do the flowers attract so many insects that seem poorly suited to pollinating them? Is this simply an unavoidable consequence of producing nectar and scent signals that appeal to many different animals? Or might the presence of trapped insects actually reduce reproductive success by blocking access to the flowers’ reproductive structures?

And, returning to where I started, what exactly is pollinating those plants on the Danish shoreline at Klint? Are they visited by the same diversity of insects as the Austrian populations, or has their rather exposed coastal environment resulted in a very different assemblage? I still don’t know the answer to that question. But it would be fascinating to find out.

One of the things I enjoy most about working on the Apocynaceae is that each new study seems to reveal another layer of complexity in this extraordinary family. Almost 40 years after I began studying their flowers and pollinators, they continue to surprise me. My thanks to Wujian and all of our colleagues for helping to unravel another part of that story.

Here’s the full reference, with a link to the open-access paper:

Xiong, W., Ollerton, J., Liede-Schumann, S., Meve, U., Wagner, H.C., You, W., Mu, J. & Dötterl, S. (2026) Generalized pollination of morphologically specialized Vincetoxicum hirundinaria (Apocynaceae, Asclepiadoideae). AoB PLANTS 18(5): plag048. https://doi.org/10.1093/aobpla/plag048

Images above (c) Wujian Xiong

Moths, wasps, hummingbirds and nectar: exploring the pollination ecology of Apocynaceae in Argentina

One of the things that has fascinated me throughout my career is the extraordinary diversity of ways in which flowering plants interact with their animal visitors. Nowhere is this better illustrated than in the milkweed and dogbane family, the Apocynaceae, a group that I’ve been studying for almost 40 years.

Only last month I wrote about the remarkable pollination biology of Heterostemma ficoides, a species from Thailand that deceives fig wasps while offering a genuine breeding site to tiny flies. That was an example of an unusual pollination system involving a single species. But what happens when we look at a whole community of Apocynaceae growing together in the same habitat? Do they share pollinators, or have they evolved different ways of attracting and using animals?

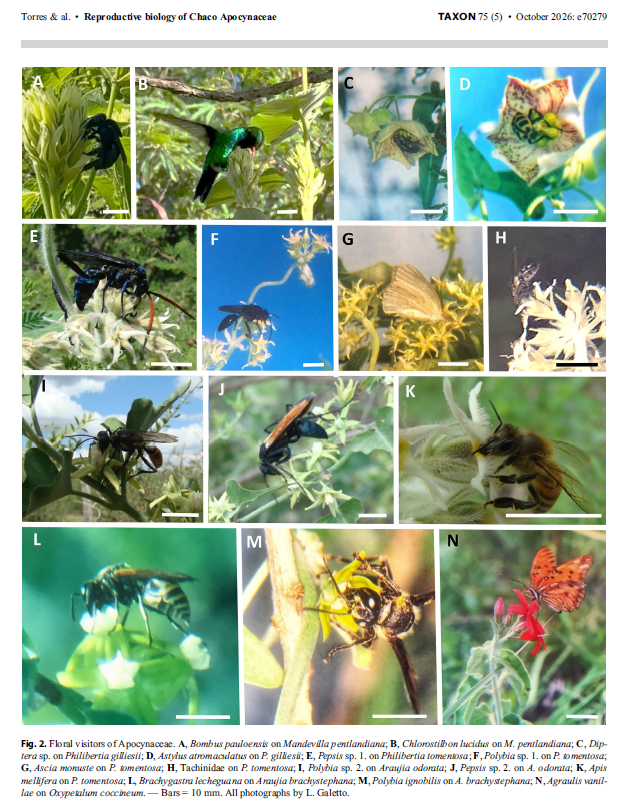
Those are some of the questions that my Argentinian colleagues Carolina Torres and Leonardo Galetto and I have addressed in a new paper just published in the journal Taxon. The study focuses on eleven species of Apocynaceae growing together in the Chaco forests of central Argentina, a region characterised by strongly seasonal rainfall and a distinctive assemblage of plants and animals.

What’s particularly interesting is that the original field observations were made by Carolina and Leonardo over three flowering seasons between 1997 and 2000. We have now brought those data together, including detailed measurements of floral nectar, and added analyses of the networks of interactions between plants and their visitors. It’s a nice example of how carefully collected field data can continue to yield new insights many years later.

Different flowers, different rewards

The eleven species represent three major evolutionary lineages within the Apocynaceae: one rauvolfioid, three apocynoids (Mandevilla species), and seven members of the Asclepiadoideae, the group formerly recognised as the separate family Asclepiadaceae.

Their flowers vary enormously in size and structure. At one extreme are the relatively small flowers of species such as Araujia, Oxypetalum and Philibertia. At the other are the large, tubular flowers of Mandevilla, including M. petraea, in which the functional floral tube is more than 10 cm long.

These differences are reflected in the nectar that the flowers produce. The three Mandevilla species generally offer relatively large quantities of nectar containing substantial amounts of sugar, predominantly sucrose. They are visited by animals capable of accessing these rewards, including long-tongued hawkmoths, bumblebees and, in the case of M. pentlandiana, hummingbirds. By contrast, most of the smaller-flowered species produce much less nectar and show greater variation in the proportions of the three main nectar sugars: sucrose, glucose and fructose.

But these relationships are not quite as straightforward as we might expect. For example, two closely related species, Araujia brachystephana and A. odorata, have rather similar-looking flowers, yet the former produces nectar dominated by sucrose while the latter produces nectar consisting almost entirely of glucose and fructose. Both are visited primarily by wasps, although A. brachystephana attracts a broader range of insects.

In other words, even closely related species living in the same habitat may differ substantially in the rewards they offer and the animals that visit them.

There’s another intriguing result concerning the tree Aspidosperma quebracho-blanco. Previous research described its flowers as deceptive, attracting visitors without offering nectar. Yet in our study we found small quantities of nectar containing mainly glucose and fructose. Does nectar production vary between populations, or were there differences in the methods used to study the flowers? It’s an interesting question that deserves further investigation.

Sharing the flowering season

The timing of flowering is another important part of this ecological story. Most of the species flowered during the warmer, wetter months, particularly December and January, with flowering often continuing for three or four months. Seed dispersal, by contrast, was concentrated mainly between February and June, when conditions become progressively drier.

This makes ecological sense. Water availability is likely to be an important trigger for flowering in this seasonal environment, while the wind-dispersed seeds of these species are released mainly during the drier part of the year. But it also means that many of the species are flowering simultaneously and potentially competing for the attention of the same animals.

One possibility is that plants avoid this competition through differences in flowering time. Another is that they coexist by attracting different groups of pollinators, or by using the same pollinators in subtly different ways. For example, two Mandevilla species may share hawkmoth visitors but place their pollen on different parts of the moth’s proboscis, potentially reducing interference between their reproductive systems.

Among the smaller-flowered asclepiads, differences in the intricate structures that attach pollen masses to visiting insects may perform a similar function. These are fascinating examples of how floral morphology can influence ecological interactions, even when the same animals visit several plant species.

What do the interaction networks tell us?

As readers of this blog will know, I’ve been interested in plant–pollinator networks for many years. One reason for analysing these networks is that they allow us to move beyond individual plant species and examine how an entire assemblage of organisms is connected.

In the Chaco study, we found a mixture of apparently specialised and generalised relationships. Some species were visited by just one major functional group, such as wasps or butterflies, while others attracted a much wider range of insects. Wasps were particularly conspicuous. Indeed, two social wasps, Polybia ignobilis and Brachygastra lecheguana, were among the visitors that connected different parts of the interaction network. The introduced western honey bee, Apis mellifera, also played a connecting role.

It’s another reminder that when we talk about pollinators, we really need to look beyond bees. Wasps, flies, moths, butterflies and other animals can be important components of these ecological communities.

One intriguing outcome of our analyses concerns the overall structure of the network. At first glance, the interactions appear to be organised into distinct groups, or modules, with particular sets of plants sharing particular sets of visitors. However, when we compared the observed network with randomly generated networks that preserved the number of interaction partners of each species, neither its modularity nor its nestedness was significantly greater than expected.

In other words, although some groups of interactions look rather specialised, there is limited statistical evidence for strong compartmentalisation within this particular assemblage. The patterns may largely reflect differences in how many partners each species has, rather than the existence of clearly separated ecological groups.

There is an important qualification here. Our network includes only eleven plant species, all from the same family, rather than the full diversity of flowering plants in the Chaco forests. A more comprehensive network might reveal additional structure that we cannot detect at this scale.

This connects rather neatly with my recent discussion of global patterns in plant–pollinator specialisation. One of the lessons from that research is that specialisation depends partly on the spatial, taxonomic and ecological scale at which interactions are examined. What looks specialised at one scale may be much more generalised at another.

I should also emphasise that this is a network of floral visitors, not necessarily effective pollinators. We recorded animals capable of contacting the reproductive structures of the flowers, and of carrying pollinaria, but that does not establish that they successfully transferred pollen between plants. As I discussed in an earlier post about what we actually mean by a pollination system, that distinction really matters.

Back to the bigger picture

For me, this study makes an interesting contribution to the broader understanding of Apocynaceae pollination ecology that my colleagues and I developed in our 2019 global review of the family’s pollination systems. In that paper, involving 75 authors, we showed that Apocynaceae exhibit an extraordinary diversity of pollination systems, with strong evolutionary and biogeographical patterns. But we also emphasised how much remains unknown, with reliable pollination information available for only a little over 10% of the family’s species. The new Chaco study adds something that large-scale reviews cannot provide on their own: a detailed picture of how related species interact with their floral visitors within the same ecological community.

There’s also a connection to our recent review of edible Apocynaceae, which also involved Carolina and Leonardo. One of the striking results of that study was how little we know about the pollination biology of many species whose fruits, seeds or other parts are used by people. Understanding how these plants reproduce is important not only from an evolutionary perspective but also for their conservation and sustainable use.

Ultimately, what I find most interesting about this new paper is the contrast between the extraordinary diversity of floral forms and rewards, and the extent to which different species can share the same visitors. Specialised flowers do not necessarily mean exclusive relationships with particular pollinators. And generalised patterns of visitation do not mean that floral morphology and nectar chemistry are unimportant. The reality is more complicated, shaped by evolutionary history, seasonality, floral structure and the behaviour of the animals themselves.

It’s also a reminder of the continuing value of detailed natural history. Large-scale databases and sophisticated network analyses are enormously useful, but they depend ultimately on people spending time in the field, watching what visits flowers, measuring nectar, and recording when plants flower and produce seeds. Sometimes those observations take decades to reach their full potential. But that doesn’t make them any less valuable.

Here’s the full reference, with a link to the paper:

Torres, C., Ollerton, J. & Galetto, L. (2026) Reproductive phenology, flower-nectar traits, and floral visitors of eleven co-occurring species of Apocynaceae from Chaco forests (Argentina). Taxon 75(5): e70279. https://doi.org/10.1002/tax.70279

Listen to Karin and I on The Gardener’s Lodge podcast: pollinators, gardening and relationships

Back in the summer, Karin and I were interviewed, one after the other, by garden designer and podcaster Mykal Hoare for his The Gardener’s Lodge podcast. Both interviews have now been released, covering rather different aspects of gardening and our relationship with the natural world.

My interview, published on 17 September, was a wide-ranging conversation about pollinators, their relationships with flowering plants, and the role that gardens can play in supporting biodiversity. We discussed everything from bees and butterflies to birds, the effects of climate change and this summer’s unusually hot, dry weather, and the perennial question of whether gardeners should favour native or non-native plants. We also talked about why providing flowers is only part of the story when it comes to conserving pollinators.

Karin’s interview, published on 1 October, approached gardening from a very different perspective. Drawing on her experience as a relationship therapist and author, she and Mykal explored how gardens and gardening can contribute to mental wellbeing, mindfulness and stronger relationships. In particular, they discussed how gardening together can reveal differences between couples, provide opportunities for communication and compromise, and strengthen our connections with nature. Apparently, our own sometimes contrasting ideas about how tidy or wild a garden should be provided some useful examples!

There’s quite a bit of common ground between the two conversations, particularly around the importance of observing and appreciating the wildlife that shares our gardens.

Some readers may remember that Karin has spoken about gardening and relationships on a podcast before, so this is an interesting continuation of that discussion.

Many thanks to Mykal for inviting us both onto the podcast and for two very enjoyable conversations!

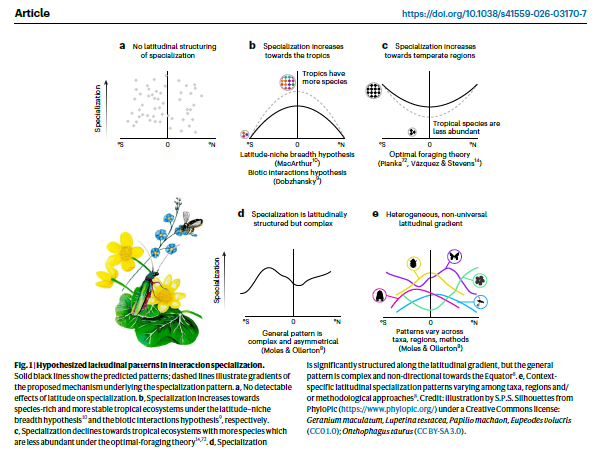
Are plant-pollinator interactions more specialised in the tropics? A new global analysis suggests that it’s complicated…

Some scientific questions have a habit of following you around for much of your career. Back in 2002, Louise Cranmer and I published a paper in the journal Oikos asking a deceptively simple question: are tropical plants more specialised in terms of their pollinators?

At the time there was a widespread assumption in ecology that interactions between species become increasingly specialised as you move from the poles towards the tropics. It’s an attractive idea which had some (quite vague) theoretical support. Tropical ecosystems contain more species, have experienced relatively stable climates over long periods of evolutionary time, and seem like just the sort of places where tightly specialised interactions ought to evolve.

The trouble was that the evidence wasn’t especially convincing, in part because it hadn’t actually been well studied. In preparing the 2002 paper, Louise and I found only a handful of empirical studies that had addressed the question, not just for plants and pollinators, but for ALL kinds of interactions.

The question of tropical specialisation has subsequently cropped up repeatedly in my research. In 2014, Angela Moles and I went considerably further and asked whether the broader claim that species interactions are stronger and more specialised in the tropics might actually be a “zombie idea” – one of those scientific notions that persists despite accumulating evidence that the reality is considerably more complicated. That guest post on the Dynamic Ecology blog was then written up as an invited paper for Biotropica see: Tropical Zombies: Moles & Ollerton (2016) is now published.

Twenty-four years after that first Oikos paper, we can now address the question with a dataset that Louise and I could scarcely have imagined in 2002. A huge international collaboration led by Sailee Sakhalkar and Robert Tropek has just published “Global patterns in plant–pollinator specialization” in Nature Ecology & Evolution.

I’m delighted to be one of the co-authors and I find the answer to the question that we posed 24 years ago to be fascinating.

More than 110,000 interactions

The scale of the new study is worth emphasising. It assembled 3,415 quantitative plant-pollinator networks from 162 studies, covering 110,571 pairwise interactions between 5,343 pollinator species and 6,126 plant species. The data span almost all of the world’s terrestrial biogeographic regions, from 43.6°S to 81°N and from sea level to more than 4,000 metres elevation.

That makes this the most comprehensive attempt yet to examine the geography of specialisation in plant-pollinator interactions. But simply throwing thousands of networks into a statistical analysis would potentially create as many problems as it solves. Different researchers study pollination networks in very different ways. Some attempt to sample whole communities, while others concentrate on particular groups such as bees, hummingbirds or particular plants.

So an important feature of this study was that we explicitly separated these different types of datasets and accounted for sampling completeness and methodological differences. We also looked separately at different functional groups of pollinators rather than assuming that bees, beetles, butterflies, moths, flies and birds should all behave in the same way. That turned out to be important in ways that we could not predict.

So, are interactions more specialised in the tropics?

The short answer is no, not in any simple sense. There is geographical structure to plant-pollinator specialisation. But there is no straightforward increase in specialisation as you approach the Equator – nor, for that matter, a straightforward decrease. Instead, the patterns are distinctly nonlinear.

Network-level specialisation and pollinator specialisation tended to peak at relatively low northern latitudes, at around 20°–30°N, close to the tropical-subtropical boundary. I find this particularly interesting as I think the subtropics have been a bit neglected as a focus of ecological research: no one ever refers to themselves as a “subtropical ecologist” and there is no Journal of Subtropical Ecology. Yet the subtropics are not simply a transitional zone between the tropical and temperate worlds. They encompass an extraordinary range of ecosystems, including deserts, Mediterranean-type vegetation, subtropical forests, and some major centres of biodiversity and endemism. This includes the distinctive habitats in Yunnan that I’m exploring during my visits to China. Perhaps we need to start thinking of the subtropics as an important biogeographical region in their own right, rather than as the ecological space between two better-studied zones?

Plant specialisation showed a different and weak hemispherically asymmetric pattern. And once individual pollinator groups were examined separately, the picture became more complicated still. Hoverflies, for example, came closest to the traditional expectation of increasing specialisation towards the Equator. Birds showed something closer to the opposite pattern, while moths did something much more complicated.

In other words, there isn’t a latitudinal specialisation gradient. There are several overlapping geographical patterns whose shapes depend upon what organisms you study and what measure of specialisation you are considering.

That conclusion feels satisfying given the arguments Angela Moles and I made ten years ago. We suggested that attempts to find a universal latitudinal gradient could obscure the fact that different groups of organisms have different evolutionary histories, physiologies and ecologies. That is very close to what emerges from this much larger analysis.

Perhaps latitude was never really the interesting variable

One of the most intriguing results is what happens when we stop asking about latitude itself. We compared latitude with a suite of possible explanatory variables, including temperature, precipitation, environmental productivity, and plant and pollinator diversity. Climate generally did a better job of explaining specialisation than latitude, biodiversity or productivity. Again, however, there wasn’t a single climatic rule.

At the whole-network level, specialisation generally declined as mean annual temperature increased, which was not expected at all and runs counter to the argument that the tropics are always more specialised. Precipitation produced strongly nonlinear relationships, and plants and different pollinator groups responded differently. Birds, insects and even different groups of insects could show contrasting responses to the same climatic gradient.

There are some plausible biological explanations for these patterns. Warmer conditions may extend flowering periods and pollinator activity, creating more opportunities for species to encounter alternative partners and therefore encouraging generalisation. Colder or more seasonal environments might compress flowering and pollinator activity into shorter periods, producing tighter temporal matching between species. Rainfall adds another layer of complexity because it can influence flowering but also directly constrain pollinator activity.

These are hypotheses rather than demonstrated mechanisms, however. As we stress in the paper, these are correlational global patterns and climate covaries strongly with latitude. The results shouldn’t therefore be interpreted as demonstrating simple causal effects of temperature or rainfall.

Specialisation depends on how you look at it

There’s another connection here to research I’ve discussed previously on the blog. In work with Danish and Brazilian colleagues, for example, we showed that the apparent specialisation of plants and pollinators depends partly on the spatial scale at which interactions are examined – see Local and regional specialization in plant–pollinator networks. More recently I’ve written about why scale matters when analysing plant-pollinator networks.

And earlier this year, our global analysis of plant-pollinator interactions in gardens found that the factors explaining species richness were not necessarily those explaining interaction specialisation: Global drivers of plant-pollinator interaction specialization in gardens.

There’s also a nice connection to another study that I wrote about here in 2022. With Pablo Gorostiague and Pablo Ortega-Baes, I looked specifically at whether cactus pollination systems become more specialised towards the tropics. Our answer was yes and no: tropical cacti were visited by somewhat fewer pollinator species, but there was no latitudinal pattern in the number of functional pollinator groups that they used. As I wrote at the time, the answer depended on what we meant by “specialised”: Are cactus pollination systems more specialised in the tropics? A new study suggests yes…and no!

All of these studies point towards a similar conclusion: “specialisation” is not a single, fixed property of an ecological community. What we detect depends upon biological scale, geographical scale, the organisms being considered, and how the interactions have been sampled. That doesn’t make specialisation meaningless. Quite the opposite, it means we need to be precise about what sort of specialisation we’re talking about and at what scale.

The new global study puts that result into a much broader context. Different groups really can display different geographical patterns of specialisation, so studies focused on a particular lineage aren’t necessarily contradicting one another when they produce different answers. They may simply be measuring different pieces of a much larger ecological puzzle.

Why does any of this matter?

Specialisation is not just an esoteric property of ecological networks. It affects how plants and pollinators partition resources, how species coexist, how communities are assembled, and potentially how ecological systems respond when species disappear.

That becomes especially important in a changing climate. Our results suggest that changing temperature and rainfall regimes could restructure plant-pollinator networks, but they are unlikely to do so uniformly. Different pollinator groups and different parts of the world may respond in very different ways. Highly specialised interactions may also be particularly vulnerable to changes in phenology or the loss of interaction partners. Predicting the consequences therefore requires us to move beyond simple statements about “tropical” and “temperate” ecosystems.

For me, though, there is also a broader lesson here about how science progresses. In 2002, Louise Cranmer and I questioned whether the available evidence really supported the assumption that tropical plant-pollinator interactions were more specialised. Fourteen years later, Angela Moles and I argued that the wider claim about stronger and more specialised tropical interactions might be a zombie idea. Now, with more than 110,000 plant-pollinator interactions available for analysis, the answer is much clearer. Latitude matters; climate matters; the identity of the organisms matters; and ecology, as usual, refuses to obey a simple rule.

My particular thanks to Sailee and Rob for the monumental efforts they made to pull this work together, and cudos to all of the co-authors who helped to make the study possible.

Want to conserve birds and mammals? Then conserve their insects – our new paper in Nature Reviews Biodiversity sets out the details

It’s sometimes easy to forget quite how much of the living world depends upon insects.

That might seem an odd thing for someone who has spent much of his career studying insects and their relationships with plants to say. But conservation, ecological research, and public interest are still disproportionately focused on vertebrates: the birds, mammals, reptiles, amphibians and fishes that most people think of when they hear the word “wildlife”.

Yet those animals exist within ecological networks in which insects are frequently central players, not walk-on extras. A new review that I’ve co-authored with Rob Cooke, Eliza Grames, Chris Elphick and 18 other colleagues, published in Nature Reviews Biodiversity, tries to bring together what we know about those relationships – if you follow this link it’s free to read:

Cooke, R., Grames, E.M., Ollerton, J. et al. (2026) The importance of insect biodiversity for vertebrates. Nature Reviews Biodiversity DOI: 10.1038/s44358-026-00201-w.

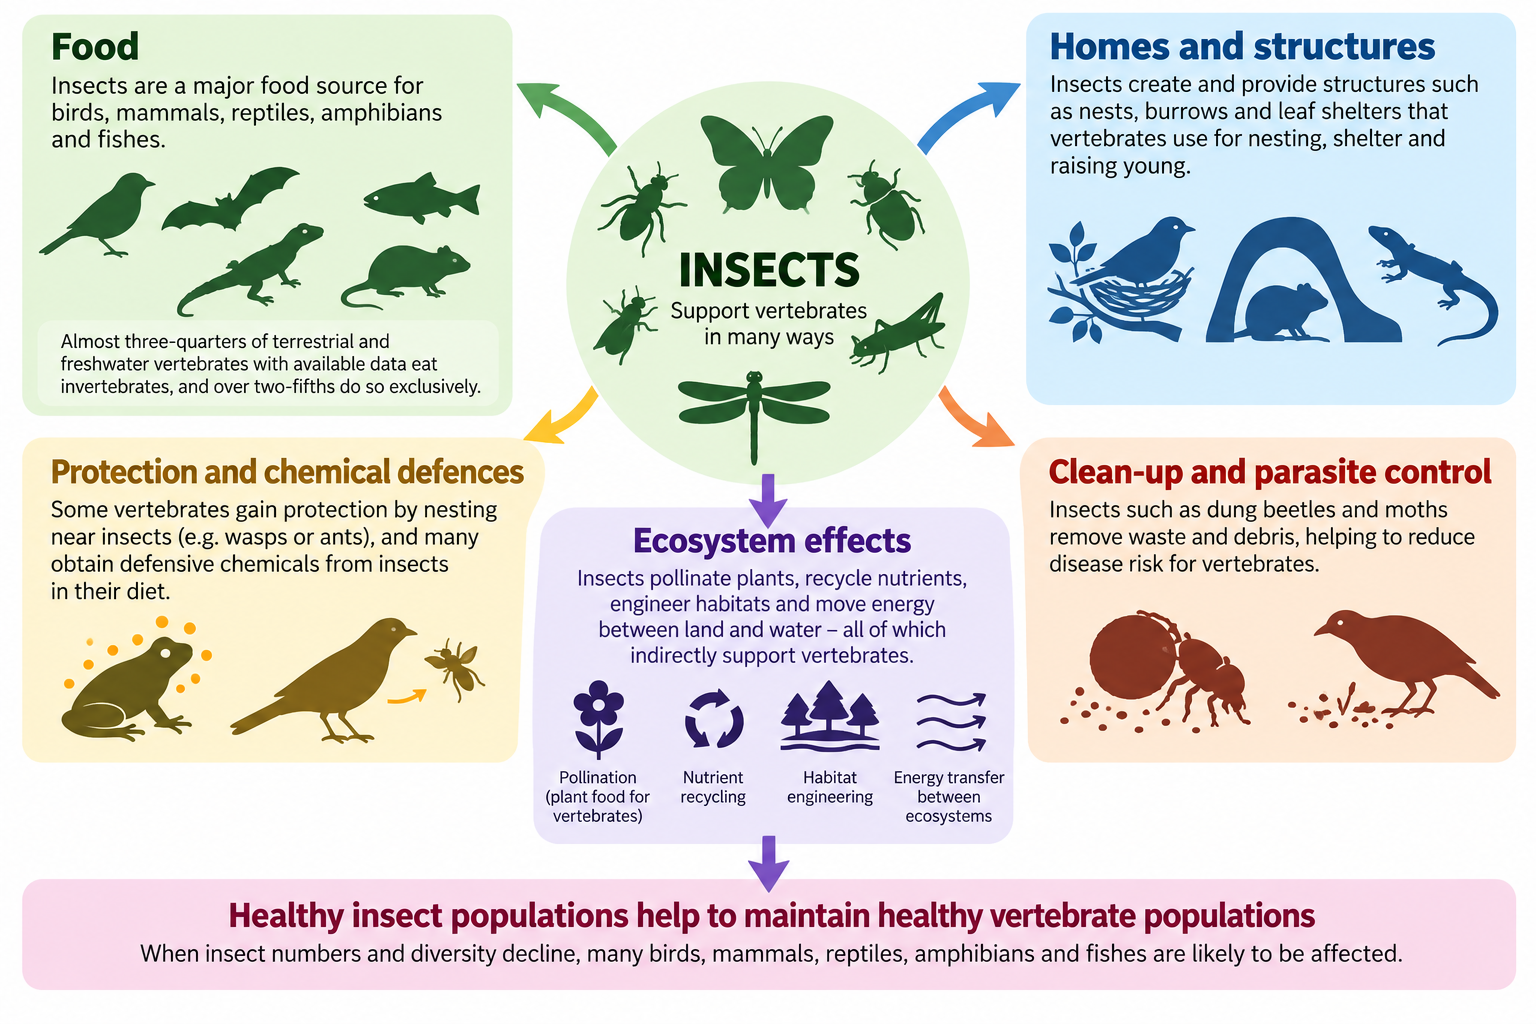
The starting point is food, and the numbers are striking. We assembled diet information for 19,750 species of terrestrial and freshwater vertebrates. Of those for which data are available, 73% eat invertebrates and 44% eat them exclusively. That alone ought to give us pause when thinking about the consequences of insect declines.

But one of the things that I particularly enjoyed about writing this review is exploring with colleagues how food is only the beginning of the story. All of us involved in it, I think, learned just as much as we contributed.

Much more than something to eat

The relationships between insects and vertebrates are extraordinarily varied, and some are wonderfully unexpected. Termite mounds and ant nests provide nesting sites, refuges and places to lay eggs for mammals, birds, reptiles and amphibians. Some bats use cavities created by beetle larvae. Birds incorporate insect and spider silk into their nests. Other birds deliberately nest close to wasps or ants, apparently gaining protection from predators.

Then there are the chemical relationships. Poison frogs obtain many of their defensive alkaloids from the insects and other arthropods that they eat. Some snakes acquire defensive toxins from fireflies. Birds, mammals, reptiles and amphibians engage in various forms of “anting” or anointing, applying ants and other invertebrates to their bodies, probably for a variety of functions including parasite control.

Insects can even provide sanitation services. Beetles remove vertebrate dung and can thereby reduce the survival of parasites, while moths living in the nests of some birds consume faeces and other organic debris. There is fossil evidence that similar relationships involving feather-feeding beetles occurred in dinosaur nests during the Cretaceous.

One of the figures in the paper brings together examples from around the world, and is worth spending some time exploring. There are chimpanzees applying insects to wounds, parrots nesting in termite mounds, geckos “milking” honeydew from planthoppers, frogs sheltering in ant nests, herons using insects as fishing bait, and much more. Ecological interactions are rarely dull!

Insects connect ecosystems

There is also a much bigger ecological story within this review, because insect relationships with vertebrates move enormous quantities of energy and nutrients through ecosystems. Aquatic insects emerge from streams and lakes and become food for terrestrial animals; terrestrial insects fall into rivers and feed fishes. In some forest birds, aquatic insects can provide more than a quarter of their energy budget, rising seasonally to 50–90%. Conversely, terrestrial invertebrates can provide approximately half of the annual energy budget of freshwater fishes.

And then there are the indirect effects. As readers of this blog will know, a lot of my research and writing is related to plant pollination, but insect pollination doesn’t just matter to plants. When an insect pollinates a plant whose fruits or seeds are subsequently eaten by a bird or mammal, the insect is indirectly supporting that vertebrate too.

One striking example concerns figs. Fig trees depend upon their tiny agaonid wasp pollinators, while figs themselves are eaten by at least 1,274 species of birds and mammals. Remove the wasps and the consequences potentially propagate far beyond the insects and plants themselves.

This is something I’ve discussed from a different direction in my book Birds & Flowers, where the focus is largely on birds as pollinators rather than insects supporting birds, though all nectar-feeding birds also consume insects. But the broader lesson is the same: species do not exist independently of the ecological relationships that sustain them. I’ve written previously about some of the extraordinary diversity of these pollination relationships on this blog, including in my post on the limits to pollinator diversity.

What happens if the insects disappear?

This brings us to the more difficult question addressed by the review. There is now substantial evidence that insect abundance, biomass and diversity are changing, although, as I’ve argued on this blog before, the magnitude, geography and taxonomic extent of those changes need to be discussed carefully rather than reduced to simplistic claims of an impending “insect apocalypse”.

Nevertheless, widespread changes in insect populations inevitably raise the question of what happens to the vertebrates that depend upon them. Here the evidence becomes surprisingly patchy.

There are good reasons to expect effects: a meta-analysis of 125 studies, for example, found strong positive relationships between insect prey availability and bird reproductive success and chick condition. European insectivorous birds declined by 13% between 1990 and 2015 while omnivorous bird populations remained stable. There are also examples involving bats, small mammals and other groups.

But demonstrating that declining insects actually caused a particular vertebrate population to decline is much harder. Insects and vertebrates can respond simultaneously to habitat destruction, pesticides, climate change and other pressures, making cause and effect difficult to disentangle.

That’s an important distinction. Ecology is full of plausible stories; demonstrating the causal links is another matter. There are nevertheless cases where dependence on particular insects is difficult to ignore. The Critically Endangered Mountain Pygmy Possum in Australia depends heavily on Bogong Moths, whose numbers have crashed. The probable extinction of the Eskimo Curlew has likewise been linked partly to the disappearance of the Rocky Mountain Locust, formerly an important component of its diet.

A surprisingly large gap in our knowledge

Perhaps the thing that surprised me most while working on this review was how poorly documented many insect–vertebrate interactions remain. Even something as apparently straightforward as “what insects does this bird eat?” often turns out not to have a satisfactory answer. Studies may report prey simply as “invertebrates”, “arthropods”, or “insects”, with little or no taxonomic resolution. Birds are much better studied than most other vertebrates, yet detailed quantitative diet information is still available for only a small fraction of species.

Non-feeding relationships are even more scattered through the literature. This is part of what ecologists call the “Eltonian Shortfall“: our incomplete knowledge of who interacts with whom in nature.

One conclusion of the review is therefore that we need much better ways of recording these interactions: common data standards, better taxonomic resolution, long-term monitoring, experiments, larger databases, and greater collaboration between entomologists and vertebrate ecologists. Citizen science, computer vision, metabarcoding and environmental DNA all have potentially important roles to play.

There is also a plea here for something rather unfashionable: natural history. Observations of animals eating, nesting, sheltering, grooming and otherwise interacting with insects are not trivial anecdotes. Properly documented and brought together, they are the raw material from which larger ecological patterns emerge.

Conserving relationships, not just species

For me, one of the broader messages from this review is that conservation needs to pay much more attention to what I’ve referred to in the past as the “biodiversity of species interactions“.

We naturally talk about conserving species and habitats. But an ecosystem is not merely a list of species occupying the same place. It is also the vast network of feeding, pollination, seed dispersal, decomposition, competition, parasitism, facilitation and other interactions connecting those species.

Lose enough of those connections and an ecosystem can change profoundly even before many species have disappeared. That has a very practical implication: insect conservation is also vertebrate conservation. If we want landscapes that support healthy populations of birds, bats, amphibians, fishes and other vertebrates, maintaining abundant and diverse insect communities is not an optional extra. It is part of the ecological infrastructure upon which those animals depend. And, as our review makes abundantly clear, we have probably only begun to understand the full extent of that dependence. That’s why nature conservation policies and regulations, such as Biodiversity Net Gain (BNG) in England for instance, need to look carefully at their implications for insects and other invertebrates.

Finally, I’d like to thank all of the contributors to this paper for working so diligently on the review. It’s an output from the Vertebrates and Insects Working Group, which was formed by the Status of Insects Research Coordination Network – check out the website and get involved!

A century of genetic erosion in a British bumblebee – a new study just published

Back in 2022 I wrote about a project in which I’d been involved with colleagues at the Natural History Museum, Imperial College London and several regional museums. We were using preserved bumblebees to ask a deceptively simple question: what can insects collected decades ago tell us about the environmental changes that their populations have experienced?

The first papers from that project showed two important things. One found increasing signs of developmental stress in the wings of museum bumblebees over the course of the 20th century, associated particularly with hotter and wetter conditions. The other demonstrated that it was possible to recover and sequence surprisingly good-quality DNA from insects collected more than a century ago, in some cases using just a single leg.

At the time I wrote that this opened up the possibility of looking at how the genomes of bee populations had changed through time. Well, we’ve now done it.

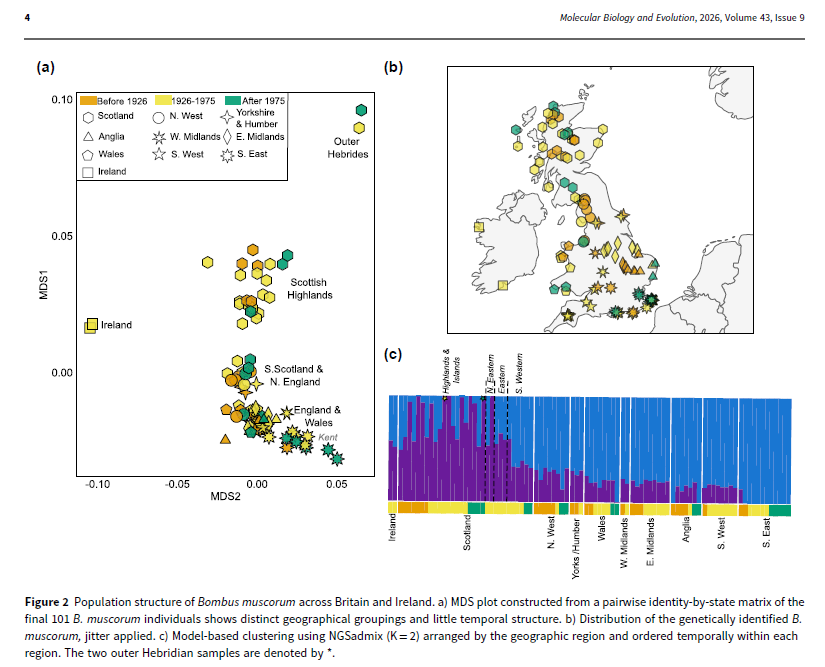
Published this week in Molecular Biology and Evolution, our new study focuses on the Moss Carder Bumblebee (Bombus muscorum), a beautiful species of flower-rich grasslands, heaths, marshes and coastal habitats. Once much more widespread across Britain, it is now largely concentrated in Scotland and the Scottish islands, with scattered populations surviving around the coasts of England and Wales.

Led by Victoria Mullin, the team generated whole-genome data from museum specimens collected between 1894 and 2019. The results provide a rather sobering picture of what has happened inside these bee populations as their geographical distribution has contracted.

Comparing bees collected before 1926 with those collected after 1975, we found about a 25% reduction in genome-wide genetic diversity. Looking at the full time series gives the same basic message: heterozygosity declined progressively through the 20th century, with no obvious sign of recovery.

That matters because losing a species is not the only way that biodiversity can decline. Long before extinction, populations can become smaller and more isolated and begin to lose genetic variation. That variation is part of the raw material that allows populations to respond to environmental change, disease and other challenges.

There was also a striking geographical pattern. In England and Wales, the amount of the genome occurring in long stretches of homozygosity increased by about 186% – in other words, almost threefold. These “runs of homozygosity” are consistent with populations becoming smaller, more fragmented and increasingly isolated from one another. Scotland showed a much weaker change, reflecting the fact that B. muscorum remains considerably more widespread there.

Importantly, however, the population structure is not simply “Scottish bees versus English bees”. The genomic data reveal a broad north-to-south gradient across Britain – what population geneticists call isolation by distance – rather than a set of sharply separated populations. That has implications for conservation because fragmentation may be breaking what was once a more continuously connected population into increasingly isolated regional groups.

There’s another interesting connection here with work that I published with colleagues more than a decade ago. In our 2014 Science paper we used historical records to show that Britain had lost 23 species of bees and flower-visiting wasps, with the fastest rate of extinction occurring from roughly the late 1920s to the late 1950s. We argued that large-scale changes in British agriculture, beginning just after the First World War, were an important part of that story.

The new study is looking at genetic change within a surviving species rather than the disappearance of whole species and it cannot pin that change on a single cause. But the parallels are difficult to ignore. The loss and fragmentation of flower-rich habitats associated with agricultural intensification is a likely contributor, alongside pesticides, climate change and other environmental pressures. The genomic erosion appears to have accumulated progressively across much of the same century in which Britain’s pollinator landscapes were being radically transformed.

One unexpected finding was also a useful warning about museum data. Of the 130 specimens originally labelled as Bombus muscorum, genetic analysis showed that 29 (almost a quarter) were actually two other, morphologically similar bumblebee species. Museum collections are extraordinarily valuable, but identifications cannot always simply be taken at face value, particularly for difficult groups. Genomics provides both a historical record and a way of checking the identity of the specimens supplying that record.

And that brings me back to what I think is one of the wider messages of this whole project: natural history collections are not dusty archives of dead organisms, they are biological time series.

A pinned bumblebee collected more than a century ago preserves information about where a species occurred, what environmental stresses it experienced, and, as we can now show, the genetic diversity of the population from which it came. Combined with modern genomic techniques, the millions of insects sitting in museum drawers around the world represent an extraordinary resource for understanding biological change.

The conservation message for the Moss Carder Bumblebee itself is fairly straightforward. Protecting the remaining populations is not enough if they become progressively smaller and more isolated. Restoring large areas of suitable, flower-rich habitat and reconnecting populations should help maintain population sizes and gene flow. More interventionist approaches such as translocation or assisted gene flow may eventually have a role, but would need careful assessment because of issues such as local genetic structure and disease transmission.

Four years ago, when I blogged about the first papers from this project, I finished with the idea that museum genomics might allow us to understand how insect populations had adapted, or failed to adapt, to a century of environmental change. We now have part of that answer. And it shows that beneath the visible contraction of a species’ range, another quieter form of biodiversity loss can be taking place: the erosion of diversity within its genome.

The paper is open access and you can download a copy here:

Mullin, V.E., Merchant, H.N., Arce, A.N., Nash, W. et al. (2026) Museum specimens reveal the genomic consequences of long-term population decline in an insect pollinator. Molecular Biology and Evolution 43: 1-11.

Fake figs, fooled wasps, and another extraordinary Apocynaceae pollination system

One of the things I love about working on the milkweed and dogbane family (Apocynaceae) is that it has an apparently inexhaustible capacity to produce strange and wonderful interactions with animals. Just when you think that the family’s pollination biology has yielded most of its surprises, along comes something like this.

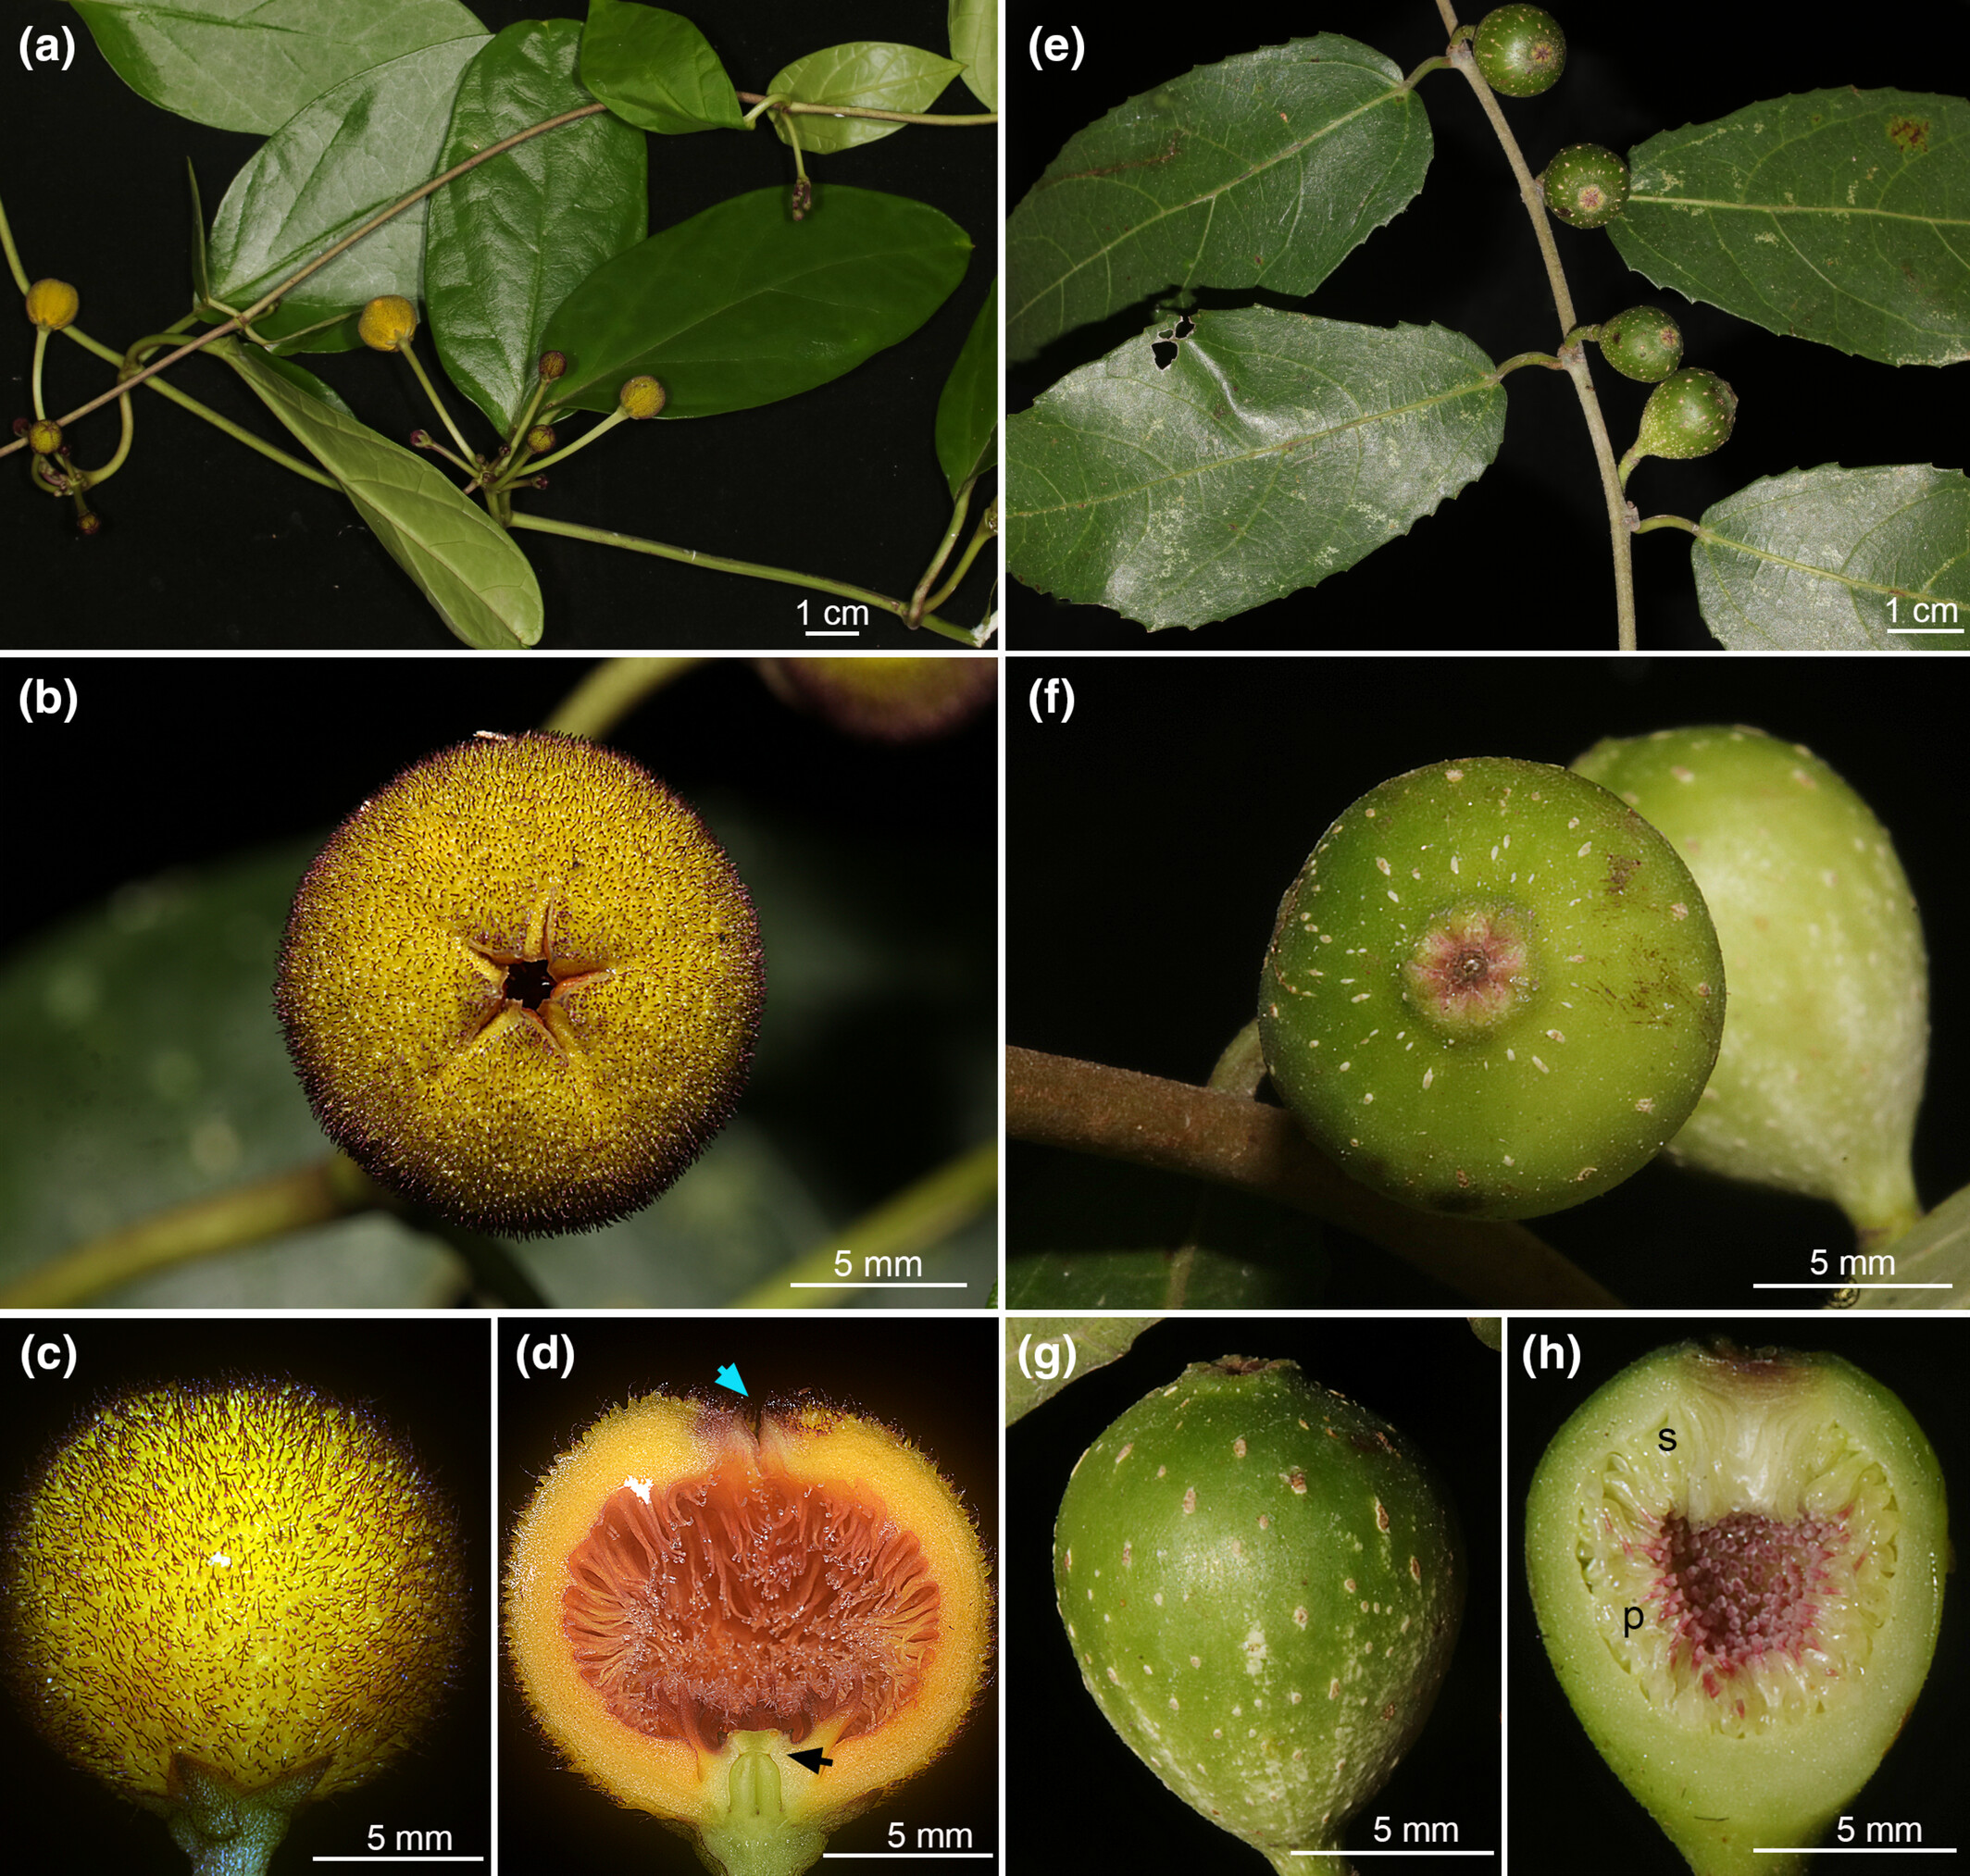
A paper just out in New Phytologist, led by Aroonrat Kidyoo, describes the pollination of Heterostemma ficoides, an unusual climbing plant from northern Thailand. The title rather neatly gives away the story: “Fake figs, fooled fig wasps and rewarded phorid flies: brood-site mimicry and mutualism in Heterostemma ficoides (Apocynaceae)”.

And “fake figs” is not journalistic exaggeration, as you can see from the photos above, which are taken from the paper. The flowers of H. ficoides are globose, fleshy structures, about 1.5–2 cm across, with a small opening at the top. Superficially they look remarkably like the enclosed inflorescences (the syconia) that we normally call figs. Indeed, when the species was first described in 2019, its resemblance to a fig was obvious enough to inspire the name ficoides: fig-like. But looking like a fig is only the beginning of the story.

Fooling one of nature’s most specialised pollinators

The relationship between figs (Ficus) and their tiny agaonid wasps is one of the classic examples of an intimate plant–pollinator mutualism. Female fig wasps locate receptive figs using their scent, squeeze through the tiny opening or ostiole, and pollinate the enclosed flowers while attempting to reproduce inside. These relationships can be remarkably specific, in some cases representing rare examples of one-to-one plant-pollinator interactions.

So it was genuinely surprising to discover female Kradibia fig wasps entering flowers of Heterostemma ficoides. These wasps normally pollinate Ficus heterophylla, not an Apocynaceae, and the authors believe that nothing comparable, i.e., a fig wasp being fooled into visiting a completely unrelated flowering plant, has previously been documented. I have to concur, this relationship is (so far) unique.

The authors have neatly demonstrated that the deception of these wasps is not simply visual. The chemical bouquet produced by H. ficoides is closer to that of receptive Ficus heterophylla figs than it is to the flowers of its relative H. siamicum. More importantly, behavioural experiments showed that Kradibia wasps were significantly attracted to the scent of open H. ficoides flowers, though not to unopened flower buds. In other words, the plant seems to switch on its misleading olfactory advertisement at just the right time.

Once inside, however, the wasps discover that they have made a serious mistake. They wander around probing the inner surface, searching for egg-laying opportunities that simply aren’t there. Some die inside the flower, although more than 80% of observed individuals managed to get out again, and often went on to visit another Heterostemma flower.

In the process, pollen can be transferred between flowers, but as in other members of the Asclepiadoideae, Heterostemma does not dust its visitors with loose pollen grains. Instead, pollen is packaged into pollinia which become attached to the legs of the fig wasps.

So from the fig wasp’s perspective this is straightforward deception: the plant promises a breeding site that doesn’t exist, and the flowers get pollinated in return. But that is only half of the system.

The flies are not being fooled by the fake fig

The most important pollinator of H. ficoides appears to be a tiny phorid fly in the genus Megaselia, and its relationship with the plant is quite different. Female Megaselia enter the flowers and lay their eggs there. Mating may even take place on the flower beforehand. Their larvae then develop inside the fallen flowers, eventually completing their development in the decomposing floral tissue on the forest floor. For these flies the promise made by the flower is therefore an honest one: this really is a brood site.

Pollinaria become attached to the flies’ mouthparts, then the flies carry them to another flower, where pollen can be deposited. Interestingly, Megaselia are also important pollinators of some species of the related Ceropegia in Africa (both genera are members of the tribe Ceropegieae).

This creates an ecological combination that is one of the most distinct examples of a “bimodal pollination system” that I’m aware of, in which the same flower operates simultaneously as a brood-site mutualism and as a brood-site deception, involving two completely distinct groups of insects.

Back to our 2019 Apocynaceae review

For me, there is a satisfying connection here with the large review of Apocynaceae pollination systems that we published in Annals of Botany in 2019: The diversity and evolution of pollination systems in large plant clades: Apocynaceae as a case study. Aroonrat Kidyoo, lead author of this new study, was also one of the large international team involved in that paper.

We assembled usable pollination information for 567 species (a bit more than 10% of the family) and found an extraordinary diversity of interactions. About 73% of the species for which we had information were associated predominantly with a single broad pollinator group, whether bees and wasps, butterflies and moths, flies, beetles or birds. However, about 7% of the species had distinct bimodal pollination systems, such as bee + butterfly. Whether this is an unusually high proportion for such a family is currently unclear as there are few comparative statistics.

One of our broader conclusions from the study was that this interaction diversity was not randomly scattered across the Apocynaceae evolutionary tree. Pollination systems show strong phylogenetic structure and some transitions between pollinator types have occurred much more readily than others. The new Heterostemma study puts some wonderfully detailed natural history onto that much larger evolutionary picture.

Aroonrat and her colleagues suggest that Heterostemma ficoides may represent a shift away from the more open, nectar-producing flowers found in other parts of the genus. In section Oianthus, to which H. ficoides belongs, the flowers have become progressively more closed. In the extreme case represented here, the result is a globose chamber entered through a small opening, nectar production has apparently disappeared, and the plant has moved towards brood-site pollination by flies and deception of fig wasps.

Whether that evolutionary scenario survives a proper phylogeny and detailed pollination studies of the remaining species is an obvious question for the future. As the authors themselves acknowledge, both are currently lacking. But it is exactly the sort of transition that our 2019 study suggested we should be looking for.

And what does any of this have to do with eating Apocynaceae?

Quite a lot, in a roundabout way. Earlier this year my colleagues and I published another large synthesis of the family, this time asking a very different question: which Apocynaceae do people eat?

We documented 440 edible species, spread widely across the evolutionary tree of the family. That sounds like a lot, although statistically Apocynaceae are actually under-represented among the world’s food plants, probably in part because the family is so well endowed with toxic and pharmacologically active chemistry.

One point that emerged strongly from that work was that our knowledge of how those useful plants reproduce is remarkably incomplete. Many edible Apocynaceae are harvested for their fruits and seeds, which of course ultimately means that successful reproduction matters. Yet for most of those species we still know little or nothing about their pollinators.

That matters if we are serious about conserving wild food plants or developing some of them as future crops. You cannot fully understand the biology of a fruit-producing plant without understanding how the flowers get pollinated in the first place.

There are no Heterostemma species documented in our edible-plant study (though it appears that we missed one – see the comment below), so H. ficoides is not some promising new food species. But that isn’t my point. Rather, this new research is a reminder of just how much biological complexity can lie behind the production of an Apocynaceae seed. And we still know the pollination biology of only a fraction of this enormous family.

That, perhaps, is the broader lesson from all three papers. Large databases and family-wide syntheses are valuable because they reveal general patterns and, equally importantly, the gaps in our knowledge. But filling those gaps still depends on researchers spending time watching individual plants and individual insects, dissecting flowers, rearing larvae and asking exactly what the animals are doing. Sometimes what they find is stranger than anyone would have predicted.

Join me for “Pollinator Conservation: Threats and Opportunities” in Bedfordshire on Tuesday 15th September

Bedfordshire Natural History Society (BNHS) has invited me to give a talk on the theme of “Pollinator Conservation: Threats and Opportunities” at Maulden Village Hall (MK45 2DP) on Tuesday 15th September. It starts at 8pm and non-members are encouraged to attend.

More details are available at the BNHS web site.

I’ll have signed copies of my books available to purchase, so if you’re in the area, please do come along.