
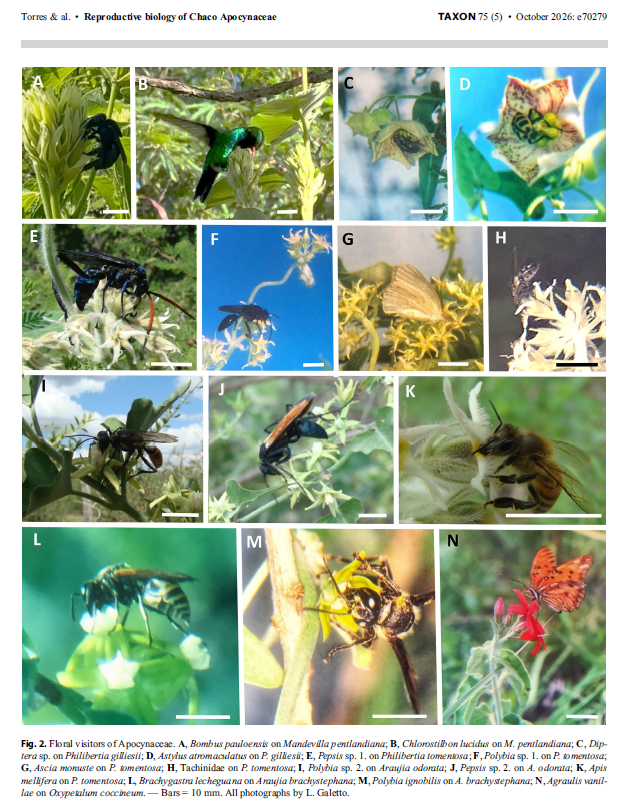
One of the things that has fascinated me throughout my career is the extraordinary diversity of ways in which flowering plants interact with their animal visitors. Nowhere is this better illustrated than in the milkweed and dogbane family, the Apocynaceae, a group that I’ve been studying for almost 40 years.
Only last month I wrote about the remarkable pollination biology of Heterostemma ficoides, a species from Thailand that deceives fig wasps while offering a genuine breeding site to tiny flies. That was an example of an unusual pollination system involving a single species. But what happens when we look at a whole community of Apocynaceae growing together in the same habitat? Do they share pollinators, or have they evolved different ways of attracting and using animals?
Those are some of the questions that my Argentinian colleagues Carolina Torres and Leonardo Galetto and I have addressed in a new paper just published in the journal Taxon. The study focuses on eleven species of Apocynaceae growing together in the Chaco forests of central Argentina, a region characterised by strongly seasonal rainfall and a distinctive assemblage of plants and animals.
What’s particularly interesting is that the original field observations were made by Carolina and Leonardo over three flowering seasons between 1997 and 2000. We have now brought those data together, including detailed measurements of floral nectar, and added analyses of the networks of interactions between plants and their visitors. It’s a nice example of how carefully collected field data can continue to yield new insights many years later.
Different flowers, different rewards
The eleven species represent three major evolutionary lineages within the Apocynaceae: one rauvolfioid, three apocynoids (Mandevilla species), and seven members of the Asclepiadoideae, the group formerly recognised as the separate family Asclepiadaceae.
Their flowers vary enormously in size and structure. At one extreme are the relatively small flowers of species such as Araujia, Oxypetalum and Philibertia. At the other are the large, tubular flowers of Mandevilla, including M. petraea, in which the functional floral tube is more than 10 cm long.
These differences are reflected in the nectar that the flowers produce. The three Mandevilla species generally offer relatively large quantities of nectar containing substantial amounts of sugar, predominantly sucrose. They are visited by animals capable of accessing these rewards, including long-tongued hawkmoths, bumblebees and, in the case of M. pentlandiana, hummingbirds. By contrast, most of the smaller-flowered species produce much less nectar and show greater variation in the proportions of the three main nectar sugars: sucrose, glucose and fructose.
But these relationships are not quite as straightforward as we might expect. For example, two closely related species, Araujia brachystephana and A. odorata, have rather similar-looking flowers, yet the former produces nectar dominated by sucrose while the latter produces nectar consisting almost entirely of glucose and fructose. Both are visited primarily by wasps, although A. brachystephana attracts a broader range of insects.
In other words, even closely related species living in the same habitat may differ substantially in the rewards they offer and the animals that visit them.
There’s another intriguing result concerning the tree Aspidosperma quebracho-blanco. Previous research described its flowers as deceptive, attracting visitors without offering nectar. Yet in our study we found small quantities of nectar containing mainly glucose and fructose. Does nectar production vary between populations, or were there differences in the methods used to study the flowers? It’s an interesting question that deserves further investigation.
Sharing the flowering season
The timing of flowering is another important part of this ecological story. Most of the species flowered during the warmer, wetter months, particularly December and January, with flowering often continuing for three or four months. Seed dispersal, by contrast, was concentrated mainly between February and June, when conditions become progressively drier.
This makes ecological sense. Water availability is likely to be an important trigger for flowering in this seasonal environment, while the wind-dispersed seeds of these species are released mainly during the drier part of the year. But it also means that many of the species are flowering simultaneously and potentially competing for the attention of the same animals.
One possibility is that plants avoid this competition through differences in flowering time. Another is that they coexist by attracting different groups of pollinators, or by using the same pollinators in subtly different ways. For example, two Mandevilla species may share hawkmoth visitors but place their pollen on different parts of the moth’s proboscis, potentially reducing interference between their reproductive systems.
Among the smaller-flowered asclepiads, differences in the intricate structures that attach pollen masses to visiting insects may perform a similar function. These are fascinating examples of how floral morphology can influence ecological interactions, even when the same animals visit several plant species.
What do the interaction networks tell us?
As readers of this blog will know, I’ve been interested in plant–pollinator networks for many years. One reason for analysing these networks is that they allow us to move beyond individual plant species and examine how an entire assemblage of organisms is connected.
In the Chaco study, we found a mixture of apparently specialised and generalised relationships. Some species were visited by just one major functional group, such as wasps or butterflies, while others attracted a much wider range of insects. Wasps were particularly conspicuous. Indeed, two social wasps, Polybia ignobilis and Brachygastra lecheguana, were among the visitors that connected different parts of the interaction network. The introduced western honey bee, Apis mellifera, also played a connecting role.
It’s another reminder that when we talk about pollinators, we really need to look beyond bees. Wasps, flies, moths, butterflies and other animals can be important components of these ecological communities.
One intriguing outcome of our analyses concerns the overall structure of the network. At first glance, the interactions appear to be organised into distinct groups, or modules, with particular sets of plants sharing particular sets of visitors. However, when we compared the observed network with randomly generated networks that preserved the number of interaction partners of each species, neither its modularity nor its nestedness was significantly greater than expected.
In other words, although some groups of interactions look rather specialised, there is limited statistical evidence for strong compartmentalisation within this particular assemblage. The patterns may largely reflect differences in how many partners each species has, rather than the existence of clearly separated ecological groups.
There is an important qualification here. Our network includes only eleven plant species, all from the same family, rather than the full diversity of flowering plants in the Chaco forests. A more comprehensive network might reveal additional structure that we cannot detect at this scale.
This connects rather neatly with my recent discussion of global patterns in plant–pollinator specialisation. One of the lessons from that research is that specialisation depends partly on the spatial, taxonomic and ecological scale at which interactions are examined. What looks specialised at one scale may be much more generalised at another.
I should also emphasise that this is a network of floral visitors, not necessarily effective pollinators. We recorded animals capable of contacting the reproductive structures of the flowers, and of carrying pollinaria, but that does not establish that they successfully transferred pollen between plants. As I discussed in an earlier post about what we actually mean by a pollination system, that distinction really matters.
Back to the bigger picture
For me, this study makes an interesting contribution to the broader understanding of Apocynaceae pollination ecology that my colleagues and I developed in our 2019 global review of the family’s pollination systems. In that paper, involving 75 authors, we showed that Apocynaceae exhibit an extraordinary diversity of pollination systems, with strong evolutionary and biogeographical patterns. But we also emphasised how much remains unknown, with reliable pollination information available for only a little over 10% of the family’s species. The new Chaco study adds something that large-scale reviews cannot provide on their own: a detailed picture of how related species interact with their floral visitors within the same ecological community.
There’s also a connection to our recent review of edible Apocynaceae, which also involved Carolina and Leonardo. One of the striking results of that study was how little we know about the pollination biology of many species whose fruits, seeds or other parts are used by people. Understanding how these plants reproduce is important not only from an evolutionary perspective but also for their conservation and sustainable use.
Ultimately, what I find most interesting about this new paper is the contrast between the extraordinary diversity of floral forms and rewards, and the extent to which different species can share the same visitors. Specialised flowers do not necessarily mean exclusive relationships with particular pollinators. And generalised patterns of visitation do not mean that floral morphology and nectar chemistry are unimportant. The reality is more complicated, shaped by evolutionary history, seasonality, floral structure and the behaviour of the animals themselves.
It’s also a reminder of the continuing value of detailed natural history. Large-scale databases and sophisticated network analyses are enormously useful, but they depend ultimately on people spending time in the field, watching what visits flowers, measuring nectar, and recording when plants flower and produce seeds. Sometimes those observations take decades to reach their full potential. But that doesn’t make them any less valuable.
Here’s the full reference, with a link to the paper:
Torres, C., Ollerton, J. & Galetto, L. (2026) Reproductive phenology, flower-nectar traits, and floral visitors of eleven co-occurring species of Apocynaceae from Chaco forests (Argentina). Taxon 75(5): e70279. https://doi.org/10.1002/tax.70279

